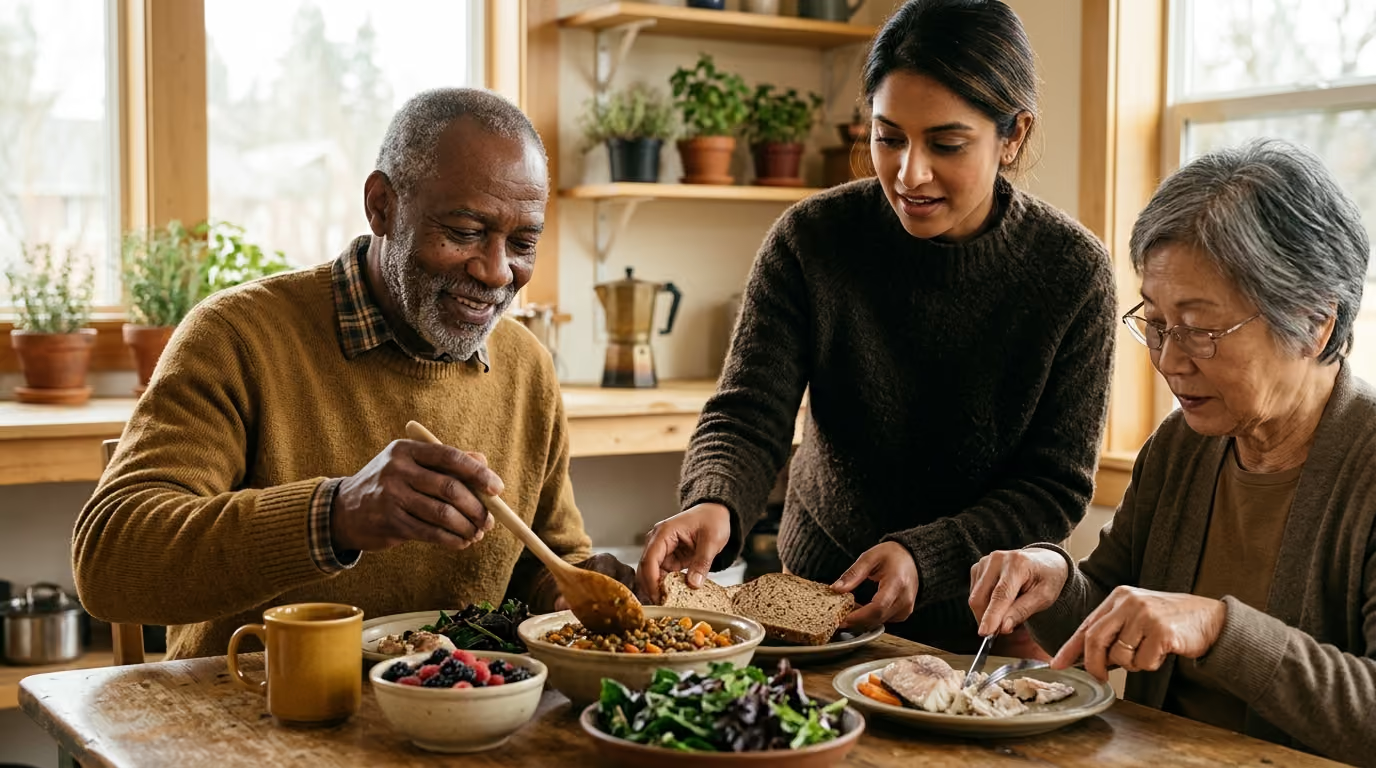
Eating a protein-rich meal activates cellular growth pathways that build vital muscle mass while simultaneously influencing biological aging and long-term metabolic health.


The mechanistic target of rapamycin, commonly known as mTOR, is a central nutrient-sensing kinase that coordinates cellular growth, metabolism, and protein synthesis. It is not an on-off switch for human longevity, nor is it a toxic cellular byproduct of eating dietary protein. Instead, this signaling pathway functions as an intracellular processing hub that weighs nutrient availability, energetic status, oxygen levels, and growth signals before directing the cell to build new structures or recycle old ones.
Longevity science has placed intense focus on this pathway over the past two decades. In preclinical model organisms ranging from yeast to rodents, dampening mTOR signaling consistently extends lifespan and delays the onset of aging-related pathology. At the same time, clinical nutrition research demonstrates that activating mTOR signaling in human skeletal muscle is essential for preserving physical strength, stimulating muscle protein synthesis, and preventing sarcopenia.
These twin observations create a biological tension. Restricting protein or calories can lower growth signaling and promote cellular cleanup, but it can also accelerate muscle wasting, weaken immune defenses, and increase frailty in older adults. Understanding how diet shapes this pathway requires looking past simplistic headlines. This resource examines the biological mechanisms of mTOR, the differences between its core protein complexes, what animal and human trials actually demonstrate, and the unavoidable physiological trade-offs between growth and cellular maintenance.
The mechanistic target of rapamycin is an evolutionarily conserved serine and threonine protein kinase. It belongs to the phosphoinositide 3-kinase-related kinase family and operates inside eukaryotic cells. Rather than measuring a single input, the pathway integrates multiple environmental cues to determine whether conditions are favorable for cell growth and division.
Upstream inputs feed continuously into this sensor. When circulating amino acids are elevated, particularly branched-chain amino acids like leucine, specialized protein complexes recruit the kinase to the lysosomal membrane. At the same time, growth factors such as insulin and insulin-like growth factor 1 signal through the PI3K and AKT cascade. This cascade relieves internal cellular brakes on the pathway.
When energy is abundant, the kinase drives downstream anabolic actions. It stimulates the translation of messenger RNA into functional proteins by phosphorylating downstream targets like p70S6 kinase 1 and the eukaryotic translation initiation factor 4E-binding protein 1. It also promotes lipid synthesis, nucleotide generation, and mitochondrial metabolism.
When nutrients are scarce, the cell shifts its priorities. A high ratio of AMP to ATP activates adenosine monophosphate-activated protein kinase, known as AMPK. Active AMPK places a direct molecular brake on growth signaling. Under these conditions, the kinase ceases its inhibitory phosphorylation of the ULK1 complex, allowing autophagy to proceed. Autophagy is the lysosome-dependent recycling system through which cells clear damaged organelles, misfolded protein aggregates, and intracellular debris. You can read more about these metabolic pathways in our guide to cellular health and metabolism.
The kinase does not act alone inside the cell. It functions as the catalytic core of two distinct multi-protein complexes known as mTOR Complex 1 (mTORC1) and mTOR Complex 2 (mTORC2). These two complexes have different structural components, respond to different upstream signals, and control completely different downstream biological programs.
mTORC1 is defined by the presence of the scaffolding protein Raptor, along with mLST8 and PRAS40. Raptor acts as an essential recruitment platform that presents specific protein substrates to the catalytic kinase domain. This complex is sensitive to rapamycin and serves as the primary metabolic sensor that responds directly to amino-acid concentrations, growth factors, oxygen availability, and cellular energy levels.
When activated, mTORC1 acts as the master driver of cell growth. Its primary jobs include:
Because mTORC1 governs both muscle protein synthesis and autophagy suppression, it is the primary focus of most nutritional research.
mTORC2 contains the defining structural protein Rictor instead of Raptor, alongside mLST8, mSin1, and Protor. Rictor alters the spatial configuration of the complex, making mTORC2 insensitive to acute, short-term exposure to rapamycin. While mTORC1 is acutely regulated by fluctuating amino-acid levels, mTORC2 responds primarily to growth factor signaling through phosphoinositide 3-kinase pathways.
The primary function of mTORC2 is to phosphorylate and fully activate protein kinase B, also known as AKT, specifically at its Ser-473 residue. This phosphorylation event is critical for downstream insulin signaling, glucose uptake, and cell survival programs. Additionally, mTORC2 regulates the actin cytoskeleton, which determines cell shape, motility, and structural integrity.
Conflating these two complexes creates significant confusion in aging discussions. Broad statements about turning down the entire pathway ignore the fact that chronic disruption of mTORC2 can impair insulin sensitivity, disrupt lipid metabolism, and trigger unwanted side effects. Understanding these distinct pathways is central to longevity nutrition and supplement research.
Dietary protein intake is the most direct physiological way humans stimulate mTORC1. When protein is ingested, digestive enzymes break it down into peptide fragments and free amino acids. These amino acids enter the bloodstream and are transported into muscle cells, where they act as signaling molecules that initiate the muscle protein synthesis cascade.
Not all dietary amino acids stimulate growth signaling equally. Essential amino acids, which the human body cannot synthesize internally, provide the primary trigger for translation initiation. Among the essential amino acids, the branched-chain amino acid leucine serves as the most potent biochemical trigger for mTORC1 activation in skeletal muscle tissue.
Inside the cell, specialized sensor proteins known as Sestrins monitor intracellular leucine concentrations. When leucine binds to Sestrin2, it releases an inhibitory complex called GATOR2. This event allows a family of small GTPases, known as Rag GTPases, to load GTP and bind to Raptor. This interaction physically translocates mTORC1 to the surface of the lysosome. Once at the lysosome, another regulatory protein called Rheb provides the final catalytic activation step.
Arginine acts through a parallel sensing mechanism involving the CASTOR1 protein and the lysosomal transporter SLC38A9. Together, leucine and arginine signal that the raw building blocks for new tissue are present inside the cell.
The muscle-building response to dietary protein changes across the human lifespan. In young, healthy individuals, a modest intake of high-quality protein easily triggers mTORC1, stimulates downstream initiation factors, and raises the fractional synthetic rate of muscle tissue. In older adults, this physiological response often becomes blunted, a condition known in gerontology as anabolic resistance.
Anabolic resistance means that an older muscle requires a higher concentration of intracellular essential amino acids to achieve the same level of pathway activation and protein synthesis seen in younger muscle. Several mechanisms contribute to this blunting, including reduced muscle perfusion, altered amino-acid transporter abundance, elevated systemic inflammation, and physical inactivity.
Because of anabolic resistance, older adults may face progressive loss of muscle mass, quality, and physical performance if protein intake is kept too low. For deeper insights into these physiological shifts, explore our resources on the biology of aging and longevity science.
To overcome anabolic resistance, nutritional researchers developed the leucine threshold hypothesis. This model suggests that a single meal must provide a specific minimum amount of leucine to fully recruit mTORC1 to the lysosome and maximize the acute muscle protein synthesis response.
However, acute muscle protein synthesis measurements reflect only short-term cellular physiology. They capture the immediate rate at which muscle incorporates labeled amino acids over several hours. They do not automatically predict whether an individual will gain muscle mass or improve physical strength over six months or two years.
A randomized controlled trial in adults aged 65 and older with low muscle mass or strength demonstrated this gap clearly. Participants received 3 grams of leucine combined with 10 grams of protein twice daily for six months. Despite the mechanistic plausibility of leucine-driven signaling, the trial found no significant improvements in appendicular lean mass, knee-extensor strength, handgrip strength, physical performance battery scores, or long-term muscle protein synthesis rates. Pathway activation in an acute setting is a necessary physiological step, but it is not interchangeable with durable clinical outcomes.
While muscle researchers view mTORC1 activation as essential for tissue preservation, geroscience researchers often view chronic overactivation of the pathway as a potential driver of aging biology. This hypothesis is supported by decades of experimental research in short-lived model organisms.
The longevity rationale for suppressing this pathway originated in genetic screens of model organisms. In Saccharomyces cerevisiae (budding yeast), Caenorhabditis elegans (nematode worms), and Drosophila melanogaster (fruit flies), genetic mutations that reduce the expression or catalytic activity of the pathway lead to consistent, reproducible extensions in median and maximum lifespan.
In rodents, pharmacologic inhibition using the compound rapamycin yields similar results. The National Institute on Aging Interventions Testing Program demonstrated that feeding rapamycin to genetically heterogeneous mice, even when started in middle age, significantly extends lifespan in both males and females. These studies established mTOR suppression as one of the most robust pharmacologic life-extension interventions known in mammalian preclinical biology.
Preclinical research suggests several biological mechanisms through which downregulating mTORC1 may delay age-related physiological decline:
However, all of these mechanisms must be viewed through an evolutionary lens. In wild conditions, downregulating growth pathways during periods of nutrient scarcity allows an organism to pause reproduction and divert scarce resources toward somatic preservation until food becomes available. Whether chronically imposing this state through extreme human dietary restriction produces identical life-extension benefits remains unproven.
Translating preclinical longevity findings to human nutrition requires evaluating human clinical trials rather than relying solely on rodent models. While rodents often spend their lives in pathogen-free cages with continuous access to food, humans live in complex environments where immune challenges, physical activity demands, and age-related muscle loss play decisive roles in survival.
The most rigorous randomized controlled trial evaluating sustained energy restriction in non-obese humans is the Comprehensive Assessment of Long-term Effects of Reducing Intake of Energy (CALERIE) Phase 2 study. This multi-center trial randomized 218 healthy adult participants to either a 24-month calorie-restricted diet or an ad libitum control diet.
The CALERIE trial found significant improvements in several cardiometabolic endpoints, including reductions in resting blood pressure, improvements in lipid profiles, enhanced insulin sensitivity, and lower circulating systemic inflammatory markers like high-sensitivity C-reactive protein.
To test whether caloric restriction affected biological aging rates, researchers analyzed blood samples from CALERIE participants using DNA methylation algorithms. An analysis utilizing the DunedinPACE algorithm, an epigenetic clock designed to measure the current pace of biological aging from blood DNA methylation patterns, reported an approximate 2% to 3% reduction in the pace of biological aging in the calorie-restricted cohort relative to controls.
However, this finding must be interpreted with appropriate scientific restraint. Other established epigenetic algorithms, including the PhenoAge and GrimAge biological clocks, showed no statistically significant differences between the intervention and control groups. More importantly, an alteration in an epigenetic surrogate marker is not direct evidence that human lifespan was lengthened. Surrogate biomarkers provide valuable research hypotheses, but they do not prove clinical life extension.
Some longevity hypotheses suggest that humans should specifically restrict protein, rather than total calories, to keep growth signaling low. However, high-quality human evidence directly linking chronic protein restriction to extended lifespan is lacking. Most human trials on low-protein diets have been short in duration, evaluating acute changes in urea excretion, kidney filtration parameters, or fasting insulin levels rather than long-term clinical healthspan.
Observational epidemiological studies examining protein intake and human mortality yield highly mixed, context-dependent results. In younger and middle-aged adults, very high intakes of animal protein are sometimes correlated with higher cardiometabolic risks, although these findings are frequently confounded by overall diet quality, fiber intake, and lifestyle factors. In older cohorts, however, higher protein intake is consistently associated with preserved lean body mass, superior physical function, lower fracture risk, and decreased mortality from falls and infectious disease.
Because dietary restriction can be challenging to maintain and carries nutritional risks, researchers have turned to pharmacological agents like rapamycin and its synthetic analogs, known as rapalogs, to study pathway inhibition in humans.
A comprehensive systematic review evaluated 19 clinical studies examining rapamycin and rapalogs in human cohorts. The researchers investigated how pharmacological inhibition affected various organ systems and physiological aging biomarkers:
Safety data from this review highlighted clear clinical distinctions. In healthy individuals participating in short-term studies, serious adverse events were rare. However, in individuals with underlying health conditions or those receiving higher, continuous doses, inhibition was linked to higher rates of bacterial infections, stomatitis (mouth ulcers), elevated total cholesterol, increased low-density lipoprotein (LDL) cholesterol, and hypertriglyceridemia.
The Participating in Age Retro-reversal with Rapamycin (PEARL) trial represents one of the few randomized, double-blind, placebo-controlled human studies designed specifically to assess the safety and efficacy of low-dose intermittent rapamycin for age-related outcomes. The trial enrolled 114 adults aged 50 to 85 over a 48-week duration.
The study evaluated body composition, physical functioning, and various metabolic parameters across different dosing regimens. The primary endpoint of reducing visceral adipose tissue was not met across the overall study cohort. Secondary outcome analyses indicated improvements in lean tissue mass and self-reported pain measures in a specific female subgroup receiving 10 mg weekly, while the low-dose intermittent protocol was characterized as relatively well-tolerated over the 48-week period.
These findings originated from a clinical preprint report, requiring cautious interpretation until validated through long-term peer-reviewed replication. Secondary outcomes in single demographic subgroups cannot be treated as proven clinical efficacy for the broader population. Human pharmacology confirms that the pathway can be modulated medically, but it does not demonstrate that taking a prescription inhibitor extends human lifespan.
The central biological mistake in popular longevity discussions is framing mTOR as a binary choice: good versus bad, or activated versus suppressed. Living biology relies on dynamic balance, tissue-specific regulation, and appropriate timing.
Skeletal muscle is not just a tool for movement. It serves as the primary metabolic sink for blood glucose disposal, an active endocrine organ that secretes signaling myokines, and a crucial amino-acid reservoir that the immune system draws upon during severe infection or physical trauma.
Loss of muscle mass and functional strength, clinically termed sarcopenia, is a major predictor of physical disability, nursing home admission, hip fractures, and all-cause mortality in older adults. Sacrificing muscle maintenance by severely restricting protein intake to keep growth signaling low carries immediate, clinically proven health risks. While basal autophagy is essential for cellular quality control, cells do not require total starvation to execute routine maintenance. Autophagy operates continuously at basal levels and fluctuates naturally between meals and during sleep.
The immune system requires rapid, robust cell division and active protein translation to respond to biological challenges. When an individual encounters a pathogen, naive T cells and B cells must proliferate rapidly and synthesize millions of specialized immunoglobulin proteins. This expansion depends entirely on functional mTORC1 activation.
Chronic, severe downregulation of growth signaling can impair this immune expansion, leaving individuals more vulnerable to infectious disease and slowing wound repair. This trade-off is evident in organ transplant medicine, where high-dose continuous rapamycin is used specifically as an immunosuppressive agent to prevent allograft rejection.
To evaluate nutritional strategies or research studies objectively, evaluate the physiological context across five specific dimensions:
For a deeper analysis of diagnostic markers and metabolic health, consult our guide to age biomarkers and diagnostics.
Because longevity science attracts significant public interest, preliminary laboratory findings are frequently overstated. To maintain rigorous scientific objectivity, it is critical to state clearly what the current body of published evidence does not support:
For research updates on emerging clinical interventions, visit our overview of biological age testing.
Translational longevity research relies on a specific set of clinical, biochemical, and epigenetic biomarkers to evaluate how nutrition, exercise, and pharmacological agents alter metabolic signaling.
Researchers use DNA methylation algorithms to estimate cellular aging rates from blood samples:
In laboratory and muscle-biopsy research, scientists quantify pathway activation by measuring the phosphorylation status of downstream target proteins:
In human clinical trials, surrogate molecular markers must be paired with functional physical measures:
No. Eating a meal that contains protein and carbohydrates activates mTORC1, which temporarily reduces the rate of autophagy initiation in metabolic tissues like the liver and skeletal muscle. However, autophagy is not an all-or-nothing switch. Basal autophagy operates continuously inside cells at low levels to remove routine debris. As nutrients are cleared from the bloodstream and metabolized over several hours, growth signaling naturally declines, allowing autophagy rates to rise again.
Plant proteins typically contain lower concentrations of essential amino acids, particularly leucine and methionine, compared to animal proteins. As a result, a standard serving of plant protein produces a smaller, more transient activation of mTORC1 in skeletal muscle. However, if an individual consumes a larger total quantity of plant protein or combines diverse plant sources to match the total leucine content of an animal protein meal, the resulting stimulation of muscle protein synthesis is largely comparable.
Resistance exercise and dietary amino acids stimulate muscle protein synthesis through distinct but complementary mechanisms. Mechanical tension from lifting weights activates mTORC1 through intracellular mechanical sensors and lipid second messengers like phosphatidic acid, while amino acids signal primarily through lysosomal Rag GTPases. Combining resistance exercise with adequate dietary protein produces an additive effect, maximizing muscle protein synthesis and overcoming anabolic resistance far more effectively than either nutrition or exercise alone.
Time-restricted eating and intermittent fasting reduce the total daily duration of high insulin and nutrient signaling, which intermittently lowers mTORC1 activity and allows periods of higher autophagy. In human clinical trials, however, the metabolic benefits of time-restricted eating are largely driven by an unintended reduction in total caloric intake rather than unique timing effects. Controlled human trials have not yet proven that intermittent fasting extends human lifespan or produces the dramatic life extensions seen in rodent caloric restriction experiments.
Stay current with research on aging biology, biomarkers, nutrition, therapeutics, peptides and longevity technology. AgeAmaze reports what the evidence shows, where uncertainty remains and which claims still need stronger data.


Follow AgeAmaze for careful reporting on what longevity science can show today and what still needs stronger evidence.
read the Blog