Methionine restriction extends life in rodent models, but human longevity benefits remain unproven and require careful balancing against risks like sarcopenia.


Eating less of an essential nutrient sounds completely contrary to good health. In traditional nutrition science, restricting an indispensable building block leads to deficiency, stunted growth, and impaired tissue maintenance. Yet in laboratory rodents, reducing the intake of a single essential amino acid called methionine consistently extends lifespan.
This unexpected finding has made methionine restriction a major subject of interest in experimental biology. Researchers have spent decades testing how altering the balance of specific amino acids influences aging pathways. To understand these findings, we must look closely at what animal research actually demonstrates, what human trials have measured, and why selective amino acid restriction is not a validated lifestyle practice.
Evaluating this science requires looking past sensational headlines. Animal longevity studies provide vital biological clues, but they cannot be translated directly into human dietary habits. Understanding the exact boundaries between preclinical discovery and human nutritional requirements is essential for anyone following longevity nutrition and supplements research.
Nutrition interventions in aging research often sound similar, but they operate through different biological mechanisms. Methionine is an essential sulfur-containing amino acid. Because the human body cannot synthesize it from other compounds, it must come entirely from the food we eat. Methionine serves as a building block for proteins and initiates protein translation. It also acts as the primary precursor for S-adenosylmethionine, the universal methyl donor for cellular methylation reactions.
Methionine restriction refers specifically to lowering the concentration of dietary methionine while keeping other nutrients adequate. In contrast, calorie restriction involves lowering total energy intake without causing malnutrition. Protein restriction reduces the total amount of all dietary proteins. Methionine restriction isolates the effect of one specific amino acid, allowing scientists to test whether longevity gains require broad energy deficits or specific amino acid signals.
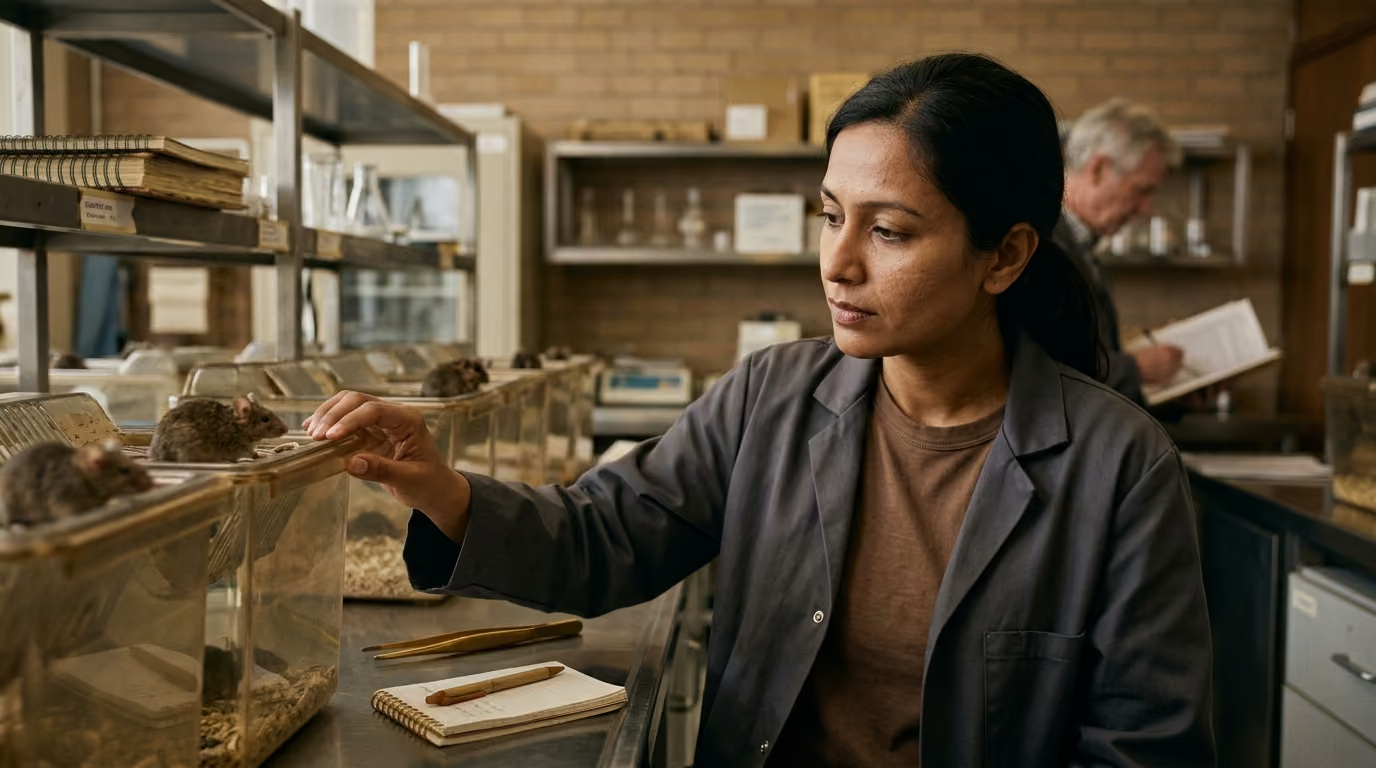
In classic rodent experiments, animals fed low-methionine diets consumed them without energy restriction. The animals were allowed to eat freely, yet they still experienced significant shifts in their lifespan and metabolic profiles. When researchers adjusted their food intake, the lifespan extensions persisted, confirming that the effect was distinct from simple caloric deprivation.
Studies also frequently look at sulfur amino acid restriction rather than methionine alone. Methionine can be converted into cysteine through the transsulfuration pathway, linking both amino acids in metabolism. Some experimental diets restrict both methionine and cysteine to observe the broader effects on sulfur metabolism. While these diets share overlapping cellular pathways, they are distinct interventions with different physiological consequences.
Understanding these distinctions prevents confusion when evaluating scientific literature. A study altering total dietary protein cannot be cited as direct evidence for methionine restriction. Similarly, studies using purified elemental diets in rodents cannot be compared directly to typical human eating patterns.
The foundational evidence for methionine restriction comes from controlled rodent experiments started in the early 1990s. In landmark experiments using male Fischer 344 rats, researchers fed one group a standard purified diet containing 0.86% methionine. The experimental group received an identical diet containing only 0.17% methionine, representing an 80% reduction in that single amino acid.
The results from these early trials were striking. Rats on the 0.17% methionine diet achieved an approximate 30% to 40% increase in median and maximum lifespan compared to controls. The restricted rats maintained lower body weights throughout their lives and showed a significant reduction in visceral fat accumulation. They also demonstrated improved insulin sensitivity and maintained youthful glucose control well into advanced age.
Intriguingly, the methionine-restricted rats did not eat less food overall. On a per-gram of body weight basis, the low-methionine animals actually consumed more food than the control animals. This hyperphagia indicated that their extended longevity was not the result of accidental calorie restriction. The animals burned more energy through increased metabolic heat production while maintaining longer functional lifespans.
Subsequent studies in various mouse strains confirmed many of these initial observations. Mice placed on low-methionine regimens showed lower rates of age-related degenerative changes and delayed onset of systemic pathology. Furthermore, studies starting the dietary restriction at 12 months of age, which corresponds to middle age in mice, still produced measurable gains in remaining lifespan.
Rodent research also documented substantial improvements in organ-specific health markers. Methionine-restricted mice displayed reduced lipid accumulation in the liver and lower levels of systemic inflammatory markers. Other studies reported a decrease in the incidence of precancerous prostate lesions in vulnerable rodent models. These healthspan outcomes confirmed that the intervention modified fundamental aspects of rodent aging biology.
However, these preclinical triumphs must be interpreted with caution. The laboratory rodents lived in sterile, pathogen-free environments with constant ambient temperatures. They received synthetic diets formulated with purified amino acid mixtures rather than intact dietary proteins. Translating an extreme 80% amino acid reduction from a caged rodent to a free-living human introduces profound biological and practical challenges.
The dramatic results seen in early rodent experiments do not represent a universal biological law. When scientists expanded methionine restriction studies to different species, strains, and genetic backgrounds, the outcomes became far more nuanced. Longevity gains from amino acid manipulation are highly sensitive to the overall genetic and dietary context.
In invertebrate models such as Drosophila melanogaster, the response to methionine restriction depends heavily on the concentration of other amino acids. Fruit flies fed low-methionine diets lived longer only when total amino acid availability was low. When researchers provided high background levels of other essential amino acids, restricting methionine failed to extend lifespan. This demonstrated that the balance across the entire amino acid profile determines the biological outcome.
Genetic variation among rodent strains also produces divergent responses to methionine restriction. While male Fischer 344 rats and certain standard mouse strains respond robustly, other genetic lines show muted or absent longevity benefits. Research involving mice with disrupted growth hormone signaling revealed that intact endocrine pathways are necessary for low-methionine diets to extend life. In mice already long-lived due to growth hormone deficiency, restricting methionine provided no additional lifespan extension.
Dietary composition plays an equally critical role in modulating the intervention. If a low-methionine diet is supplemented with small amounts of cysteine, some of the metabolic benefits in rodents are attenuated. Furthermore, restricting other specific amino acids, such as isoleucine or valine, produces metabolic shifts that overlap with, but are distinct from, methionine restriction.
These conditional outcomes demonstrate that methionine restriction is not a simple, isolated mechanism. Its effects depend entirely on species-specific life histories, metabolic rates, and precise dietary balances. An intervention that extends life in an inbred rodent strain under strict laboratory controls may have neutral or detrimental effects in an organism with different metabolic demands.
For a broader perspective on how model organisms inform the study of human longevity, readers can explore our cellular health and metabolism resources. Understanding the limits of animal modeling prevents premature assumptions about human health.
Scientists have identified several interconnected biological pathways that explain how methionine restriction alters cellular physiology in model organisms. Rather than operating through a single switch, reducing methionine intake triggers a coordinated rewiring of cellular nutrient sensing, stress resistance, and metabolic homeostasis.
The primary nutrient-sensing hub affected by methionine availability is the mechanistic target of rapamycin complex 1, commonly known as mTORC1. When intracellular methionine levels are abundant, the cell activates mTORC1, promoting protein synthesis, cell growth, and cellular proliferation. When methionine becomes scarce, mTORC1 activity decreases. This downregulation shifts cellular resources away from growth and toward somatic maintenance, protein quality control, and autophagy.
Another major endocrine pathway involved in this response is the induction of Fibroblast Growth Factor 21, or FGF21. In rodents, dietary methionine restriction rapidly stimulates the liver to produce and secrete high levels of FGF21 into the bloodstream. This hormone acts on the brain and adipose tissue to increase energy expenditure, enhance insulin sensitivity, and promote the browning of white adipose tissue.
Methionine restriction also alters mitochondrial bioenergetics and free radical generation. Animals fed low-methionine diets demonstrate reduced mitochondrial reactive oxygen species production in the liver, heart, and kidneys. This reduction in oxidative damage preserves mitochondrial membrane integrity and protects cellular lipids, proteins, and nuclear material from oxidative modifications over time.
At the cellular level, experiments using cultured human diploid fibroblasts show that restricting methionine can slow the onset of replicative senescence. Cells grown in low-methionine media maintain their replicative capacity longer than cells grown in standard nutrient concentrations. However, cellular behavior in a plastic culture dish does not replicate the complex systemic interactions of an intact human body.
These biological pathways provide compelling explanations for how diet influences cellular physiology. Nevertheless, identifying a plausible mechanism is not equivalent to proving a clinical benefit in humans. A pathway observed in rodents under extreme dietary deprivation remains an experimental observation until verified in rigorous human trials.
When we turn from animal laboratories to human clinical research, the landscape changes dramatically. There is currently no clinical evidence demonstrating that methionine restriction extends human lifespan or improves long-term healthy aging. Conducting a lifelong dietary restriction study in humans presents insurmountable logistical, ethical, and practical barriers.
Human studies on this topic have been short in duration and limited to surrogate metabolic markers. Researchers have primarily evaluated whether short-term reductions in sulfur amino acids alter biomarkers like fasting glucose, blood lipids, and body composition. These studies typically last from several weeks to a few months, involving tightly controlled liquid diets or specialized food plans.
A notable example of this research is the STAY trial, an eight-week randomized, double-blind controlled dietary intervention. The trial evaluated the physiological effects of diets containing low versus standard amounts of sulfur amino acids in adult participants. While the intervention produced minor shifts in certain metabolic markers and body weight, a subsequent analysis showed no significant impact on biological aging measures, such as epigenetic clocks.
Epigenetic clocks measure DNA methylation patterns across the genome to estimate biological age. The lack of significant change in these clocks during short-term sulfur amino acid restriction underscores the difficulty of altering complex human aging markers through brief nutritional shifts. A null finding on a surrogate biomarker does not disprove a biological effect, but it certainly offers no support for sweeping longevity claims.
Observational epidemiology provides another layer of human data, though it comes with substantial limitations. Population studies frequently examine associations between total animal protein intake, plant protein consumption, and chronic disease incidence. Some observational analyses note that diets rich in plant foods, which naturally contain lower proportions of methionine than animal proteins, correlate with lower rates of cardiovascular disease.
However, observational correlations cannot establish direct causation. Diets high in plant proteins also deliver higher levels of dietary fiber, polyphenols, potassium, and magnesium, while containing lower levels of saturated fat. Attributing the health outcomes of a plant-rich diet solely to methionine restriction ignores countless confounding lifestyle and nutritional factors.
To explore how researchers analyze population-level aging metrics, visit our coverage of longevity science and aging research news. Relying on controlled human data keeps longevity discussions grounded in reality.
Attempting to implement methionine restriction independently carries significant physiological risks. Methionine is essential for building muscle tissue, supporting immune function, and synthesizing critical molecules like glutathione, the body's primary intracellular antioxidant. Restricting this amino acid without expert clinical supervision can easily lead to inadequate total protein intake and systemic malnutrition.
The established Recommended Dietary Allowance for dietary protein in healthy adults is 0.8 grams per kilogram of body weight per day. This baseline recommendation is designed to prevent deficiency and maintain nitrogen balance in the majority of the population. It is not an arbitrary ceiling, and many individuals require higher amounts depending on their age, physical activity levels, and clinical status.
Protein adequacy is particularly crucial for older adults facing the risk of sarcopenia, the age-related loss of skeletal muscle mass, strength, and physical function. Sarcopenia is directly linked to increased risks of falls, fractures, hospitalizations, and loss of independence. As the human body ages, muscle tissue develops an anabolic resistance, meaning it requires a higher concentration of essential amino acids to stimulate muscle protein synthesis effectively.
If an older individual deliberately restricts protein or selectively cuts out protein-rich foods in an effort to lower methionine, the consequences can be severe. Muscle wasting accelerates, physical frailty increases, and recovery from acute illnesses or minor injuries becomes significantly compromised. In geriatric medicine, maintaining functional muscle mass and physical resilience takes precedence over theoretical interventions derived from rodent studies.
Several other population groups face heightened dangers from any form of amino acid or protein restriction. Pregnant and lactating individuals have increased amino acid requirements to support fetal development and milk production. Growing children, individuals recovering from surgery or traumatic injury, and anyone already struggling with low appetite or involuntary weight loss should avoid restrictive dietary regimens.
Before considering any major changes to dietary composition, it is critical to understand the foundational principles covered in our biology of aging and longevity science guides. Adequate protein intake remains a fundamental cornerstone of lifelong health.
A frequent source of confusion in longevity reporting is the conflation of intermediate biomarkers with genuine clinical outcomes. When a study reports that a dietary intervention alters a hormone level, reduces oxidative stress, or improves an enzyme concentration, these are surrogate markers. They reflect physiological activity, but they do not prove that an organism will live longer or avoid chronic disease.
In animal models of methionine restriction, scientists track numerous biomarkers, including serum IGF-1 levels, hepatic FGF21 output, glutathione concentrations, and lipid accumulation. While these measurements provide valuable insights into metabolic pathways, they are not interchangeable with lifespan data. An intervention can theoretically improve a specific metabolic marker while simultaneously causing harm to bone density, muscle mass, or immune resilience.
This distinction is even more critical in human research. In human trials, scientists cannot measure lifespan directly, so they rely entirely on short-term surrogate endpoints like insulin sensitivity, fasting lipid panels, or biological age algorithms. A favorable shift in fasting insulin over an eight-week trial demonstrates a short-term metabolic adaptation, but it does not prove that the participant will enjoy extended healthy aging over several decades.
Similarly, cellular studies provide mechanistic clues rather than practical health recommendations. Demonstrating that human fibroblasts replicate longer in a low-methionine medium shows that the cell possesses nutrient-sensing mechanisms that respond to amino acid depletion. It does not establish that a human being should attempt to deplete their own tissues of an essential amino acid.
Maintaining scientific rigor requires recognizing what the evidence does not show. Methionine restriction research does not demonstrate that humans should cut protein intake, avoid specific protein sources, or attempt to self-prescribe low-methionine diets. It remains an experimental tool used to dissect the biology of aging in laboratory settings.
For further exploration of how modern science evaluates longevity interventions, browse our comprehensive longevity science and healthy aging resources. Keeping a clear perspective on the evidence prevents unnecessary dietary risks.
To help navigate the scientific literature on dietary restriction and amino acid metabolism, the following definitions clarify key concepts discussed throughout this resource.
An amino acid that cannot be synthesized by the body from other compounds and must be obtained through the diet. Methionine is one of nine essential amino acids required for human protein synthesis and metabolic function.
A nutritional protocol in which two or more experimental feeding regimens provide the exact same total amount of dietary energy, ensuring that observed differences are not caused by variations in total calorie intake.
The primary biological methyl donor in cellular biochemistry, synthesized directly from methionine and adenosine triphosphate. It is essential for DNA methylation, histone modification, and the synthesis of neurotransmitters and cellular lipids.
A metabolic hormone produced primarily by the liver in response to specific nutritional stresses, including protein and methionine restriction. It regulates energy expenditure, glucose metabolism, and lipid homeostasis across multiple organ systems.
The progressive, age-related loss of skeletal muscle mass, strength, and physical function. Sarcopenia increases the risk of frailty, physical disability, and metabolic dysfunction in older populations.
A mathematical algorithm that estimates the biological age of a tissue or organism based on specific DNA methylation patterns across the genome. While widely used in aging research, changes in epigenetic clocks do not always correlate with clinical health outcomes.
Navigating the science of longevity requires balancing curiosity about experimental biology with practical wisdom regarding human nutrition. Methionine restriction has provided invaluable insights into the metabolic control of aging in laboratory animals, proving that specific nutrient signals can influence cellular longevity pathways independently of total calorie intake.
However, translating these laboratory discoveries into human dietary protocols is neither scientifically supported nor clinically safe. Humans possess different evolutionary adaptations, metabolic rates, and lifestyle challenges than caged rodents. For free-living adults, ensuring adequate protein intake to preserve functional muscle mass and physical vitality remains a paramount priority for healthy aging.
Scientific inquiry will continue to explore how amino acid sensing interacts with the hallmarks of aging. Until well-designed clinical trials demonstrate clear safety and efficacy in humans, selective amino acid restriction remains an intriguing area of basic science rather than an actionable personal lifestyle strategy.
Methionine restriction remains a powerful laboratory tool for understanding the biology of aging, but maintaining nutritional adequacy and preserving muscle mass are the established foundations of human health.
Stay current with research on aging biology, biomarkers, nutrition, therapeutics, peptides and longevity technology. AgeAmaze reports what the evidence shows, where uncertainty remains and which claims still need stronger data.


Follow AgeAmaze for careful reporting on what longevity science can show today and what still needs stronger evidence.
read the Blog