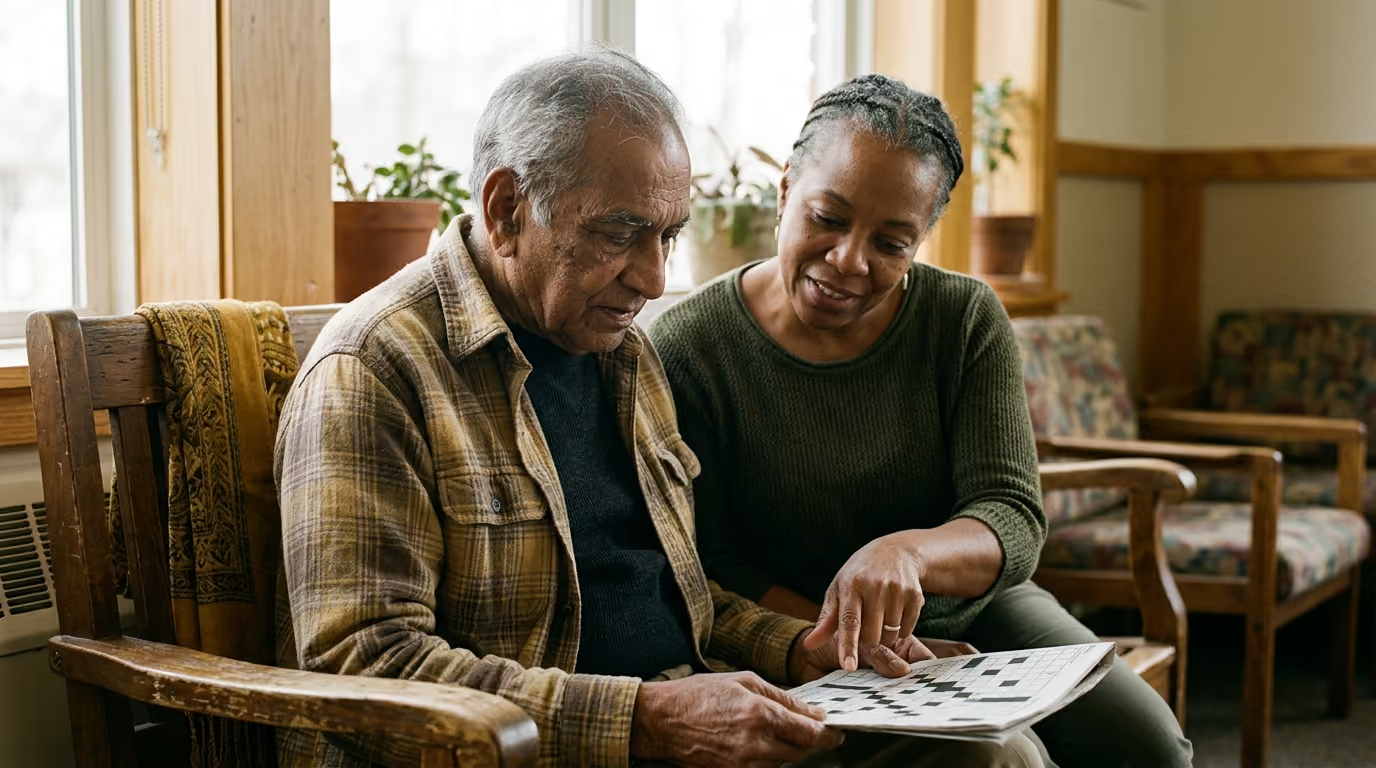
Observing physical decline in later years highlights how evolutionary pressures weaken after reproduction, allowing late-acting genetic damage and biological decay to persist.


If natural selection favors survival and reproduction, why do our bodies deteriorate as we get older? Many people search for the evolutionary root of aging, wondering whether growing old is a deliberate genetic program or a biological oversight. The definitive answer from evolutionary biology is that aging is not an active program designed to kill us. Instead, senescence happens because natural selection loses its power to protect organisms late in life.
Evolutionary biology views senescence as an age-related increase in mortality risk accompanied by a decline in physiological function and reproductive output. Across evolutionary history, external hazards like predators, pathogens, and accidents meant that very few wild organisms survived to extreme old age. Because the vast majority of reproduction happens early in adulthood, the evolutionary impact of genes that act late in life is dramatically reduced.
Understanding why natural selection does not eliminate late-life decline requires examining how selective pressures change across a lifespan. By studying demographic models, animal experiments, and human genetic datasets, researchers have established that aging stems from evolutionary trade-offs and declining selective strength. This guide provides a research-led breakdown of the evolutionary theories of aging, the empirical evidence behind them, and what these concepts mean for modern longevity science.
The foundational principle of evolutionary senescence is the age-dependent decline in the force of natural selection. In evolutionary terms, fitness is measured by the transmission of heritable genes to future generations. An organism that survives to maturity and reproduces successfully passes on its traits. However, as an organism ages, the probability of remaining alive to reproduce continuously declines due to extrinsic environmental hazards.
British biologist Peter Medawar described this phenomenon using the concept of the selection shadow. In any wild environment, external hazards such as starvation, infectious disease, harsh weather, and predation kill individuals at a steady rate. Because of this baseline mortality, a population inevitably contains far fewer older individuals than younger ones. Consequently, the cohort of older organisms contributes very little to the total gene pool of the next generation.
Biologist W. D. Hamilton later formalized this mathematically by demonstrating that the force of natural selection on survival and reproduction drops sharply after the age of sexual maturity. Natural selection acts with maximum force on mutations and traits that manifest before or during peak reproductive years. If a genetic variant causes sudden mortality in a juvenile animal, natural selection eliminates that variant almost immediately because the carrier cannot reproduce.
Conversely, if a genetic variant causes severe physiological decline or disease only after the typical age of reproduction, natural selection cannot easily remove it. The carrier has already passed the gene to offspring before the harmful effect manifests. Because the organism has already completed the bulk of its reproductive contribution, the late-acting harm remains largely invisible to natural selection. The selection shadow ensures that late-life survival receives far less evolutionary protection than early-life vigor.
The mutation accumulation theory explains how late-life harm can quietly establish itself within a species. First proposed by Medawar in 1952, this framework builds directly on the concept of the selection shadow. It suggests that genomes accumulate deleterious mutations over generations, provided their damaging effects only appear late in life.
Every generation experiences spontaneous genetic mutations. When a mutation damages essential biological processes in early life, purifying natural selection weeds it out. If a mutation disrupts cellular maintenance, bone density, or vascular integrity at an advanced age, purifying selection is too weak to purge it from the gene pool. Over thousands of generations, these neutral or weakly deleterious late-acting variants accumulate through random genetic drift.
Mutation accumulation makes a specific testable prediction about age-specific genetic variation. As an organism ages, the genetic variance in mortality and physiological failure should increase because more unpurged, late-acting mutations are expressed. Population genetic studies in model organisms have supported this prediction, demonstrating that genetic differences between individuals account for more variation in late-life survival than early-life survival.
It is critical to distinguish what this framework claims from what it does not claim. Mutation accumulation does not suggest that late-acting mutations provide any hidden benefit. It also does not argue that all aging is caused by inherited DNA sequences. Rather, it identifies an evolutionary blind spot where natural selection simply fails to keep the biological house clean once the reproductive peak has passed.
While mutation accumulation describes passive neglect by natural selection, antagonistic pleiotropy describes an active evolutionary compromise. Formulated by evolutionary biologist George C. Williams in 1957, this theory proposes that some genes control multiple distinct traits, with beneficial effects early in life but severe costs late in life.
Under the laws of natural selection, an early fitness advantage carries far more evolutionary weight than a delayed penalty. If a genetic variant improves juvenile survival, accelerates physical development, or increases early reproductive output, it confers a substantial fitness benefit. Even if that exact same variant causes arterial stiffening, cancer, or tissue degeneration at older ages, natural selection will actively favor and spread it through the population.
In this framework, aging is the biological invoice for evolutionary success in early life. Organisms do not deteriorate because natural selection wanted them to decline. They deteriorate because natural selection aggressively selected for traits that maximized early reproduction, indifferent to the late-life damage left in their wake.
Researchers exploring candidate human examples of antagonistic pleiotropy have identified several promising genetic markers. Genetic reviews analyzing human health datasets have found that specific gene variants linked to coronary artery disease are also enriched for higher lifetime reproductive success. Variants that support aggressive immune responses to clear childhood infections can promote chronic, sterile inflammation in older adults. Similarly, genes that promote rapid bone calcification during growth can contribute to calcification in blood vessels in later decades.
Human genetic studies represent observational evidence and candidate associations rather than definitive mechanistic proof. Nonetheless, antagonistic pleiotropy remains one of the most widely supported theoretical frameworks in biology of aging and longevity science resources. It explains why complex organisms inherit biological machinery that seems inherently self-destructive in late adulthood.
In 1977, biologist Thomas Kirkwood introduced the disposable soma theory, framing the evolution of aging as a problem of resource allocation. Organisms have access to finite amounts of metabolic energy gathered from their environment. An individual must divide these resources between two competing biological demands: the germline, which handles reproduction, and the soma, which encompasses all non-reproductive bodily tissues.
Every living cell continuously suffers damage from metabolic byproducts, chemical stressors, and environmental insults. Maintaining a mammalian body indefinitely requires substantial energy dedicated to DNA repair, proteostasis, antioxidant defenses, and tissue renewal. However, because extrinsic hazards will eventually kill the organism anyway, investing enough energy to maintain the soma forever represents an evolutionary waste of resources.
The disposable soma framework models an optimization strategy where the body invests just enough in somatic maintenance to keep the organism healthy through its expected reproductive window. Any additional energy is better directed toward finding mates, producing offspring, and caring for young. Somatic maintenance is deliberately imperfect, allowing molecular and cellular damage to slowly accumulate over time.
Although disposable soma shares similarities with antagonistic pleiotropy, the two concepts are distinct:
The disposable soma theory connects directly with findings in cellular health and metabolism articles. It explains why our endogenous repair enzymes, such as base-excision repair complexes and autophagic machinery, operate at levels that permit gradual physical wear and tear. Complete repair is biologically possible in principle, but evolutionary pressures did not favor paying its metabolic cost.
Evolutionary theories of aging are not just mathematical deductions; researchers have tested them directly using controlled laboratory experiments. The most famous demonstrations come from experimental evolution studies using the fruit fly, Drosophila melanogaster.
In these experiments, scientists manipulate the age at which adult flies are permitted to reproduce across dozens of generations. In lines selected for delayed reproduction, researchers collect eggs only from older females, artificially shifting the force of natural selection to later ages. Under these conditions, the selection shadow recedes, and variants that maintain late-life survival and late-life egg laying become evolutionarily valuable.
Across multiple independent laboratories, selecting for late-life reproduction consistently produces fly populations with extended lifespans. After 50 or more generations of late-life selection, experimental lines regularly exhibit average lifespan increases of 60% to 80% compared to control lines. Some experiments observe significant extensions in longevity in as few as 10 generations.
These selection experiments also illustrate the trade-offs predicted by evolutionary theory. In many long-lived fly lines, the evolution of longer lifespans is accompanied by a correlated decline in early-life fecundity. The flies lay fewer eggs during their first week of adult life in exchange for laying more eggs and surviving longer in later weeks.
However, laboratory evolution studies reveal that trade-offs are not rigid, universal rules. In some experimental paradigms, flies selected for desiccation resistance or starvation tolerance lived significantly longer without suffering measurable declines in early egg production. Preclinical animal research demonstrates that the evolutionary relationship between reproduction and somatic upkeep is flexible, depending heavily on the specific environmental stressors applied.
Evolutionary frameworks explain the broad patterns of senescence, but life on Earth exhibits immense diversity in how aging manifests. The rate of senescence is not uniform across the animal kingdom, and examining non-human species highlights important variations in evolutionary design.
Some organisms exhibit negligible senescence, meaning their mortality risk does not measurably increase with age, and their reproductive capacity does not decline. Species such as the naked mole rat, certain rockfish, and various turtles can live for decades without obvious physiological decay. A 2022 review of demographic data found that roughly 75% of 52 zoo-kept turtle and tortoise species exhibited slow or negligible senescence under captive conditions.
Other organisms show negative senescence, where mortality risk actually drops as the animal grows older and larger. This frequently occurs in species with indeterminate growth, such as certain reptiles, amphibians, and marine invertebrates. Because larger females produce exponentially more eggs, the force of natural selection on these animals increases rather than decreases as they age, favoring superior somatic upkeep throughout adulthood.
In species that experience standard senescence, including humans and fruit flies, the exponential rise in mortality does not necessarily continue indefinitely. Demographic analyses of large populations reveal that at extreme old age, the mortality rate often levels off into a plateau.
A demographic mortality plateau is an empirical observation about population statistics, not biological proof that individuals stop deteriorating. It occurs partly because the frailest individuals die off earlier, leaving a robust sub-population, and partly because the absolute force of natural selection reaches a universal baseline near zero. Recognizing mortality plateaus helps demographers interpret population curves without confusing statistical survivorship with the halting of the aging process.
Evolutionary theory and molecular biology approach aging from different analytical vantage points. Evolutionary theory addresses the ultimate question of why senescence exists as a biological phenomenon. Molecular geroscience addresses the proximate question of how physical tissues degrade inside the body. Bridging these disciplines is essential for interpreting modern longevity science.
Modern geroscience has identified several highly conserved nutrient-sensing pathways that regulate lifespan across species, including the insulin and IGF-1 signaling cascade and the mechanistic target of rapamycin (mTOR) pathway. When researchers downregulate these pathways in model organisms, the animals frequently live longer and show delayed onset of age-related diseases.
An evolutionary perspective makes sense of why these nutrient-sensing pathways exist in the first place:
Targeting these pathways with pharmacological agents or dietary protocols does not mean researchers have altered the evolutionary destiny of a species. It simply means they are modulating existing metabolic switches that evolved to manage resource allocation between growth and survival. Readers reviewing longevity research and news articles should separate an intervention's molecular mechanism from sweeping claims about rewriting evolutionary biology.
Evolutionary biology is frequently misunderstood in popular media, leading to flawed interpretations of human health and longevity. Evaluating life-extension research requires recognizing the theoretical limits and common pitfalls of evolutionary arguments.
A widespread misconception is that aging evolved as an altruistic adaptation to clear out older individuals, conserve resources, and make room for younger generations. In evolutionary biology, group selection arguments of this type have been largely rejected. Natural selection operates predominantly on individual organisms and heritable alleles. A hypothetical mutant individual that did not age would continue reproducing, quickly outcompeting individuals that sacrificed themselves for the group.
Another common assumption is that higher extrinsic mortality must always drive the evolution of faster aging. Classic evolutionary models suggested that if predators kill animals quickly, selection for somatic maintenance will inevitably collapse.
Modern evolutionary ecology demonstrates that the relationship is far more nuanced. If extrinsic hazards kill all age groups equally, or if resource competition changes population density, high extrinsic mortality can sometimes favor slower biological aging. Lifespan and the rate of senescence are distinct metrics; a population can have a short median life due to accidents while maintaining a slow rate of internal decay.
Evolutionary theory provides a lens for evaluating surrogate biomarkers of aging, such as epigenetic methylation clocks, telomere lengths, and inflammatory panels. These markers measure proximate physiological state and cellular wear.
However, a change in a surrogate biomarker does not automatically prove that an intervention has altered the evolutionary trajectory of human lifespan or reduced clinical disease endpoints. For deeper guidance on how diagnostic tools measure these changes, readers can consult biological age and testing articles to distinguish validated clinical markers from experimental proxies.
Navigating the evolutionary literature requires a clear understanding of specialized terminology. The following definitions clarify the core concepts used across evolutionary biology and longevity science:
These concepts form the vocabulary needed to critically appraise emerging studies and explore comprehensive longevity science and healthy aging resources.
Understanding the evolutionary drivers of aging helps readers evaluate emerging interventions with a grounded, scientific perspective. You can apply this evolutionary framework to assess longevity claims using the following analytical steps.
Determine the experimental system used in the study:
Never assume that an evolutionary response observed in fruit flies or mice translates directly into a human clinical outcome.
When evaluating an intervention that claims to extend lifespan or enhance vitality, ask what biological cost is being paid:
Because our biology evolved under strict resource trade-offs, artificial manipulations of major pathways frequently uncover latent biological costs.
Separate intermediate biomarkers from hard clinical outcomes:
Recognize that evolutionary biology explains why our bodies decline, but it does not prescribe a specific medical regimen. Use evolutionary principles to maintain a realistic, evidence-led mindset, avoiding sensational claims of effortless life reversal while staying informed about genuine advances in geroscience.
Stay current with research on aging biology, biomarkers, nutrition, therapeutics, peptides and longevity technology. AgeAmaze reports what the evidence shows, where uncertainty remains and which claims still need stronger data.


Follow AgeAmaze for careful reporting on what longevity science can show today and what still needs stronger evidence.
read the Blog