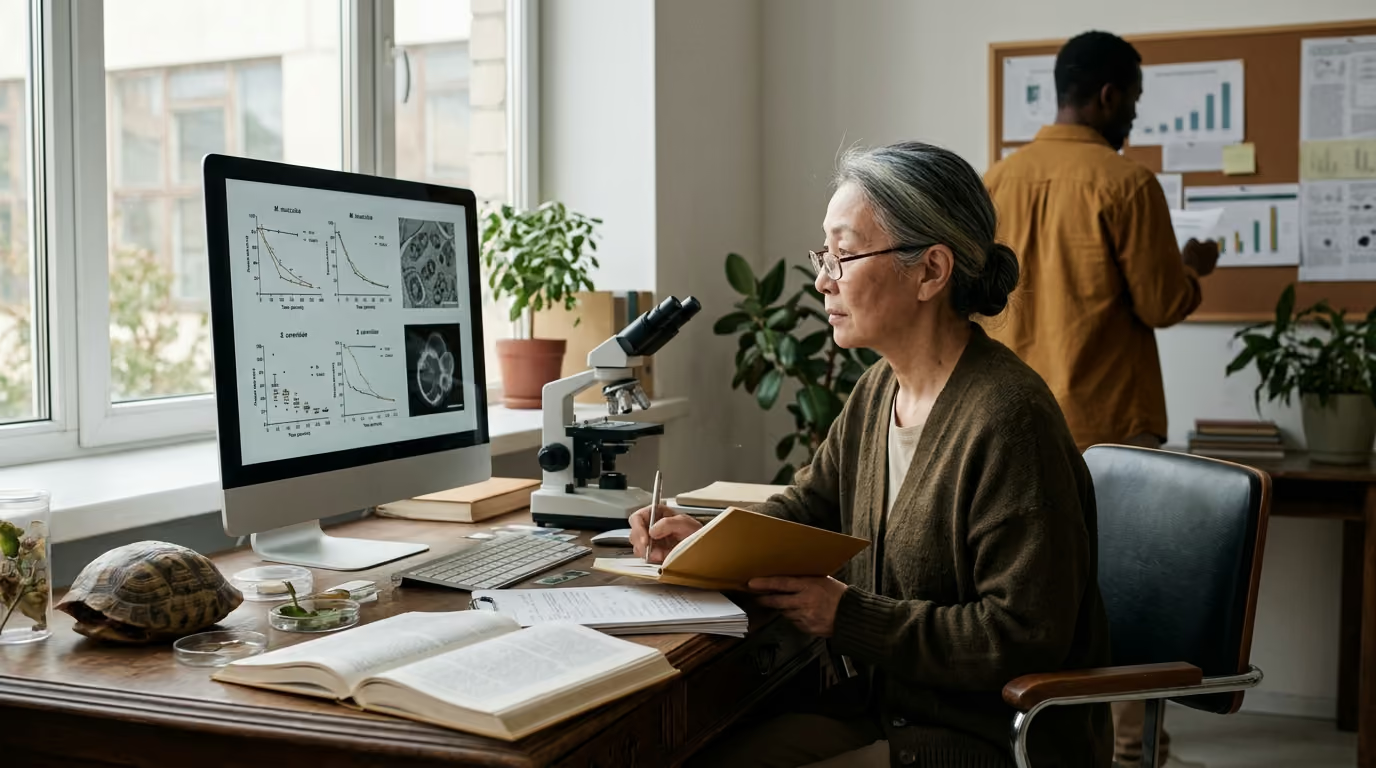
Maximum lifespan is often confused with aging rate, but comparative biology demonstrates that species follow fundamentally different demographic and cellular trajectories.


Many people search online to ask whether humans can adopt the longevity mechanisms of animals that live for centuries. Headings claiming that bowhead whales or naked mole-rats hold the hidden solution to human aging appear regularly in popular media. The plain reality is that evolution does not optimize organisms for indefinite human survival. Comparative biology provides a rigorous way to study how different species solve the challenges of cellular damage, reproduction, and tissue maintenance.
Looking across the tree of life shows that nature has generated many distinct approaches to survival. Some organisms live for centuries in freezing waters, while others survive in underground tunnels without developing tumors. Studying these animals helps researchers build hypotheses about cellular resilience and evolutionary trade-offs. However, observing a biological trait in a wild animal is never a direct recipe for a human clinical treatment.
This resource examines what comparative biogerontology reveals about the diversity of aging across species. It analyzes extreme vertebrate lifespans, tests the limits of traditional laboratory model organisms, and evaluates why interventions that extend life in mice often fail to translate directly to humans. Understanding these boundaries helps separate genuine biological discoveries from exaggerated claims.
A common misconception in longevity science is that maximum lifespan and the rate of aging are the exact same metric. Maximum lifespan represents an extreme observation of the single oldest documented individual within a population. In contrast, aging, or demographic senescence, describes how an entire population experiences changes in mortality and fertility over time. A species can possess a long maximum lifespan without necessarily aging at a uniformly slow rate across its entire life cycle.
Demographers separate the pace of life from the shape of aging. Pace refers to the absolute timescale on which life history events occur, such as the age of sexual maturity and median survival time. Shape describes whether the risk of death rises, stays flat, falls, or fluctuates as an organism grows older. Two species can exhibit the exact same shape of age-related deterioration while living on radically different timescales.
A landmark comparative review analyzing demographic data across 46 diverse species demonstrated that aging does not follow a universal trajectory across the tree of life. The survey evaluated 11 mammals, 12 other vertebrates, 10 invertebrates, 12 vascular plants, and one green alga. The researchers discovered that patterns of mortality include steeply rising trajectories, flat mortality curves, and even trajectories where mortality decreases with chronological age. The study found only a weak, statistically non-significant association between maximum lifespan and the degree of senescence (Spearman rank correlation -0.13, P = 0.362).
These findings show that species with very different absolute lifespans can share similar mortality trajectories. For example, tiny water fleas and long-lived seabirds like fulmars exhibit comparable relative shapes of demographic decline despite their vast differences in physical scale and habitat. Longevity cannot be treated as a single linear score where higher numbers automatically mean slower cellular deterioration. For a deeper look at the cellular drivers underlying these life history patterns, explore our guide to the biology of aging and longevity science.
Long-lived vertebrates offer natural case studies in extreme survival strategies. By comparing species that survive for decades or centuries with shorter-lived relatives, scientists can identify specific cellular maintenance pathways. However, studying wild and non-traditional animals comes with substantial measurement challenges.
The Greenland shark (Somniosus microcephalus) is currently recognized as the longest-lived known vertebrate. Because these deep-sea sharks lack calcified tissues that form annual growth rings, traditional aging techniques cannot determine their chronological age. Researchers resolved this problem by using radiocarbon dating on the crystalline proteins found inside the nuclei of the sharks' eye lenses. These proteins are formed during embryonic development and do not turn over during the animal's life.
An analysis of 28 female Greenland sharks yielded an estimated lifespan of at least 272 years. The largest shark in the study, measuring over five meters in length, was estimated to be approximately 392 years old. However, radiocarbon modeling carries an uncertainty interval of plus or minus 120 years for that specific individual. The study also calculated that female Greenland sharks do not reach sexual maturity until they are at least 156 years old, plus or minus 22 years.
This extreme lifespan reflects an evolutionary adaptation to deep Arctic waters, near-freezing temperatures, and a very slow metabolic rate. The shark demonstrates that vertebrate biology can maintain functional proteins and tissues for centuries. At the same time, this finding is a demographic estimate based on mathematical modeling, not a guide for manipulating human metabolic rates.
The bowhead whale (Balaena mysticetus) is the longest-lived mammal, with documented lifespans exceeding 200 years. Because whales possess vastly more cells than humans, they should theoretically face an exceptionally high risk of developing fatal cancers over a two-century lifespan. The observation that large whales do not experience higher cancer rates than small mammals is known as Peto's Paradox.
Comparative genomic sequencing has identified specific gene gains, losses, and alterations in the bowhead whale genome related to DNA repair, cell cycle control, and cancer resistance. Laboratory research on bowhead whale cells has revealed that these animals possess an enhanced capacity for repairing DNA double-strand breaks. Their cells exhibit higher repair fidelity and lower somatic mutation rates compared to cells from shorter-lived mammals.
A cold-inducible RNA-binding protein called CIRBP is expressed at unusually high levels in bowhead whale tissues and appears to play a key role in mediating this accurate DNA repair. While these molecular adaptations explain how whale cells maintain genomic integrity across two centuries, they do not prove that artificially increasing CIRBP expression in humans would safely prevent age-related diseases.
The naked mole-rat (Heterocephalus glaber) is a subterranean rodent that lives for more than 30 years in captive colonies. This lifespan is roughly ten times longer than that of a standard laboratory mouse of similar body size. Naked mole-rats maintain cardiac function, bone density, and reproductive capacity into advanced age while displaying minimal changes in age-specific mortality rates.
In laboratory settings, naked mole-rats demonstrate exceptional resistance to both spontaneous and chemically induced tumor formation. Research shows that their cells produce a unique form of high-molecular-weight hyaluronan, which triggers early contact inhibition when cells become crowded. This mechanism arrests cell division before pre-cancerous cells can organize into solid tumors.
Despite popular claims, naked mole-rats are not entirely immune to cancer. Tumors have occasionally been documented in captive individuals under specific environmental conditions. Naked mole-rats illustrate how specialized tissue environments and metabolic adaptations allow small mammals to resist common diseases of aging, but their biology reflects unique subterranean evolutionary pressures.
Much of our current understanding of genetics and cellular biology comes from laboratory organisms rather than wild animals. Organisms such as nematodes and rodents provide experimental tractability that large, long-lived animals cannot offer. Each model organism serves distinct experimental purposes and carries clear biological limitations.
The nematode worm Caenorhabditis elegans is one of the most widely used models in longevity research. It possesses an average lifespan of roughly 17 to 20 days at standard laboratory temperatures, which allows researchers to complete lifespan studies within weeks. The nematode genome is fully sequenced, its cell lineage is completely mapped, and roughly 60 to 80 percent of its genes have human homologues.
Nematodes allowed scientists to identify the first single-gene mutations that extend lifespan, particularly within the insulin and IGF-1 signaling pathways. These discoveries established that the rate of aging can be altered through targeted genetic perturbations.
However, adult C. elegans individuals consist entirely of post-mitotic somatic cells, meaning their tissues do not undergo continuous cell division or stem cell replenishment. Nematodes also lack a closed circulatory system, an adaptive immune system, and complex organs such as a brain or liver. As a result, an intervention that extends lifespan in a microscopic worm cannot be assumed to function the same way in human tissues. To understand how cellular maintenance pathways operate in mammals, read our overview of cellular health and metabolism.
Laboratory mice (Mus musculus) are mammals that share complex organ systems, immune networks, and tissue regeneration mechanisms with humans. They develop age-related pathologies including atherosclerosis, neurodegeneration, metabolic dysfunction, and solid tumors. Testing interventions in mice provides critical information about mammalian physiology that cell cultures and invertebrates cannot provide.
Despite these physiological similarities, laboratory mice have undergone decades of selective breeding in artificial environments. Standard laboratory strains, such as C57BL/6, are highly inbred and exhibit strain-specific disease susceptibilities. For example, many laboratory mouse strains die primarily from lymphomas and other hematological cancers, whereas humans face a broader spectrum of cardiovascular, metabolic, and epithelial diseases.
Furthermore, mouse metabolism operates at a vastly higher rate than human metabolism, meaning pharmacokinetics and drug clearance differ significantly. A drug that extends median lifespan in a single inbred mouse strain often fails when tested in genetically diverse populations or under different housing temperatures.
Geroscience focuses heavily on interventions that appear to work across multiple distinct species. When a compound or dietary manipulation extends life in yeast, worms, flies, and rodents, it is frequently described as universally conserved. However, closer examination reveals that these interventions often produce highly variable results depending on species, strain, sex, and dosing protocols.
Caloric restriction, defined as reducing total caloric intake without causing malnutrition, is the most thoroughly studied non-genetic longevity intervention. Research has repeatedly demonstrated that restricting calories can extend median and maximum lifespan in yeast, nematodes, fruit flies, and specific rodent strains. These effects are mediated through evolutionary nutrient-sensing pathways, including mTOR, AMPK, and sirtuins.
Caloric restriction does not produce a uniform response across all living organisms. Controlled studies have shown that dietary restriction actually shortens the lifespan of the common housefly (Musca domestica). Similar discrepancies have emerged between studies of fruit flies and Mediterranean fruit flies.
Even within mammals, caloric restriction is not universally beneficial. When the National Institute on Aging evaluated dietary restriction across recombinant inbred mouse strains, lifespan was extended in some strains, remained unchanged in others, and was significantly shortened in several genetic lines.
Non-human primate studies have also yielded nuanced outcomes. A long-term study conducted at the University of Wisconsin reported that caloric restriction improved adult survival and reduced age-related disease in rhesus macaques. Conversely, a parallel long-term study conducted by the National Institute on Aging found clear metabolic health improvements but no statistically significant extension of overall survival.
In humans, caloric restriction has never been demonstrated to extend lifespan. The Comprehensive Assessment of Long-term Effects of Reducing Intake of Energy (CALERIE) trial examined healthy, non-obese human volunteers over a two-year period. The trial measured biological aging using several surrogate biomarkers and DNA methylation algorithms.
The CALERIE analysis revealed that caloric restriction significantly slowed DunedinPACE, a blood-based biomarker measuring the pace of biological aging. However, the exact same intervention produced no statistically significant changes in other well-known epigenetic clocks, such as PhenoAge or GrimAge. This shows that surrogate biomarkers can shift without indicating a proven extension of human life.
Rapamycin, an inhibitor of the mechanistic target of rapamycin complex 1 (mTORC1), is widely considered the most robust pharmacological candidate in animal aging research. The National Institute on Aging established the Interventions Testing Program (ITP) to rigorously evaluate potential longevity compounds using genetically heterogeneous mice across three independent testing sites.
Across two decades of testing, the ITP evaluated numerous compounds. Rapamycin emerged as the only non-genetic intervention that consistently and reproducibly extended both median and maximum lifespan in male and female mice across all testing sites. Reported increases in median lifespan ranged from 14 to 26 percent in female mice and 9 to 23 percent in male mice across different dosing cohorts.
The ITP data also demonstrated that pharmacological interventions rarely affect both sexes equally. Rapamycin consistently produced larger percentage lifespan gains in female mice than in male mice. Other compounds evaluated by the ITP, such as 17-alpha estradiol and acarbose, produced substantial lifespan extensions almost exclusively in male mice.
These animal outcomes do not justify unmonitored human use. In rodents, chronic rapamycin administration is associated with notable side effects, including glucose intolerance, testicular degeneration, cataract formation, and altered immune responses. The mouse data prove that modulating mTOR signaling can alter mammalian lifespan under controlled conditions. They do not establish optimal human dosing regimens, long-term safety, or clinical efficacy in extending human life. For an analysis of experimental therapeutics in development, review our resource on longevity interventions and therapeutics.
To organize the complex biological mechanisms that contribute to cellular decline, researchers established the Hallmarks of Aging framework. Updated in 2023, this conceptual model categorizes 12 biological features associated with the aging process in mammals. These hallmarks provide a structured vocabulary for formulating hypotheses about comparative longevity.
While this framework helps organize mammalian aging research, it cannot be treated as an immutable hierarchy or a universal checklist for all living things. Primary hallmarks represent early molecular insults, antagonistic hallmarks reflect compensatory responses that turn harmful over time, and integrative hallmarks represent higher-level tissue failure.
Comparative biology demonstrates that different species handle these hallmarks in radically different ways. For example:
Observing that a long-lived animal possesses superior defenses against one hallmark does not establish that this hallmark is the sole cause of aging. Aging is an emergent, systemic process shaped by an organism's evolutionary history. Developing interventions that target a single hallmark in humans may alter specific disease risks without halting the underlying progression of biological aging.
Interpreting comparative biology requires recognizing the substantial methodological constraints that affect animal and demographic research. Overlooking these limitations often leads to premature and scientifically invalid conclusions.
Scientific knowledge about longevity is heavily skewed toward a small number of well-studied taxa. High-quality mortality and fertility data are widely available for mammals and birds because these species are economically important, commonly kept in captivity, or easily tracked in field studies. In contrast, rigorous demographic datasets for reptiles, amphibians, marine invertebrates, fungi, and bacteria remain scarce.
Statements regarding what nature allows or how aging universally functions are heavily biased by the species researchers have chosen to measure. A biological trait that appears rare may simply be unstudied in underrepresented branches of the evolutionary tree.
Lifespan measurements obtained in protected laboratory environments differ fundamentally from survival patterns in the wild. Laboratory animals live in temperature-controlled spaces with abundant food, zero predator pressure, and routine veterinary care. Under these artificial conditions, animals can survive long enough to develop degenerative pathologies that rarely occur in natural habitats.
Conversely, wild demographic studies face severe environmental noise. In nature, extrinsic mortality from predation, infection, starvation, and extreme weather often obscures intrinsic rates of cellular aging. An animal that exhibits a flat mortality curve in the wild may simply be dying from external hazards before physiological senescence can manifest.
Accurately calculating demographic rates requires large cohorts of individuals. In both human and animal studies, the number of surviving individuals decreases sharply at advanced chronological ages.
When a cohort dwindles to its final five percent of survivors, sample sizes become small and measurement error rises dramatically. Calculating mortality rates or estimating biological age from a few surviving extreme outliers frequently introduces statistical noise. Researchers must clearly distinguish between well-supported population trends and uncertain data points derived from exceptional individuals.
In human clinical research, measuring actual lifespan is impractical because studies would require seven to eight decades to complete. Consequently, researchers rely on surrogate endpoints, such as changes in epigenetic methylation clocks, inflammatory markers, or metabolic panels.
A change in a surrogate biomarker indicates that an intervention has altered a specific biological readout during the trial period. It does not prove that the intervention will prevent chronic disease, extend human healthspan, or increase maximum lifespan. Treating biomarker shifts as definitive clinical proof confuses intermediate biological signals with long-term clinical outcomes. To learn how scientists evaluate these diagnostic tools, explore our analysis of biological age testing.
Biomarkers provide the quantitative foundation for comparative longevity research and human clinical trials. Understanding what each biomarker measures, and its specific methodological limits, is critical for evaluating scientific studies.
Radiocarbon dating measures the ratio of carbon-14 to carbon-12 isotopes incorporated into non-renewing crystalline proteins inside the eye lens during embryonic development. This technique allows researchers to estimate the chronological birth year of wild vertebrates that lack calcified tissue rings, such as Greenland sharks. While highly valuable for establishing baseline lifespans in extreme species, it carries wide statistical confidence intervals and provides no information regarding cellular health or functional capacity.
These cellular assays quantify how accurately and efficiently a cell repairs severed DNA strands using non-homologous end joining or homologous recombination pathways. In comparative studies, high-fidelity double-strand break repair serves as a primary cellular marker of genomic maintenance in long-lived mammals such as bowhead whales. While this assay reveals cellular resistance to genotoxic stress in vitro, it does not measure whole-organism survival or physiological aging rates.
DunedinPACE is a blood-based DNA methylation algorithm designed to measure the current pace of biological aging rather than estimating chronological age. Developed by tracking longitudinal physiological changes across a single human birth cohort, it quantifies how rapidly an individual's organ systems are deteriorating per calendar year. In the CALERIE trial, caloric restriction successfully reduced the rate of aging as measured by DunedinPACE, though it did not alter other first- and second-generation epigenetic clocks.
PhenoAge and GrimAge are multivariate DNA methylation algorithms trained against clinical biomarkers and all-cause mortality risk. They analyze specific cytosine-phosphate-guanine (CpG) methylation sites across the human genome to assess biological risk profiles. While these clocks correlate strongly with morbidity and mortality in observational human populations, their failure to shift alongside DunedinPACE in the CALERIE trial highlights that different biological age metrics measure distinct physiological domains.
To maintain scientific rigor, researchers must clearly categorize the evidentiary level of every longevity claim. Biological insights should never be described as human outcomes when the underlying data come from animal or laboratory models.
When evaluating comparative biology and geroscience literature, readers must remain aware of explicit evidentiary boundaries. Comparative longevity studies do not establish the following:
When reading about new longevity discoveries, comparative biology studies, or emerging interventions, apply this evaluation checklist to assess the strength and reliability of the evidence.
To stay updated on rigorous, evidence-led evaluations of emerging geroscience research, visit our curated collection of longevity science and healthy aging resources.
Stay current with research on aging biology, biomarkers, nutrition, therapeutics, peptides and longevity technology. AgeAmaze reports what the evidence shows, where uncertainty remains and which claims still need stronger data.


Follow AgeAmaze for careful reporting on what longevity science can show today and what still needs stronger evidence.
read the Blog