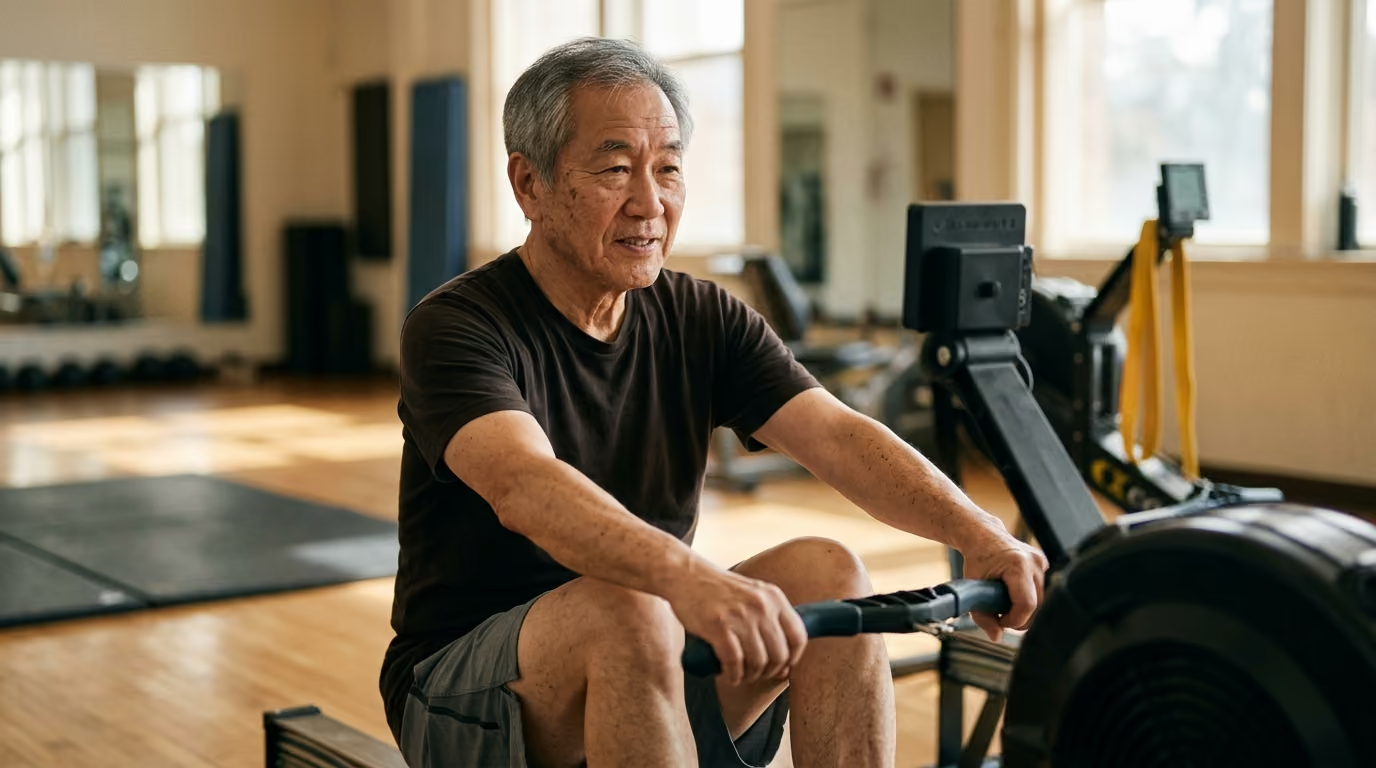
Pushing through a hard workout triggers cellular repair pathways like autophagy and antioxidant defenses that build resilience against the molecular processes of biological aging.


Many people search online to find out whether physical stress can slow the aging process. Popular discussions often claim that cold exposure, intense exercise, fasting, or heat stress will systematically rebuild the body. Others argue that stress of any kind accelerates cellular damage and promotes disease. The truth is found in a nuanced biological principle known as hormesis. This definitive guide examines the experimental evidence, the molecular mechanisms, and the strict limits of stress-induced resilience.
The central finding of hormetic biology is that biological organisms show a biphasic response to environmental exposures. A low dose of a potentially harmful stressor often triggers adaptive cellular defense pathways. A high dose of that exact same stressor causes toxicity, tissue damage, or death. In the context of longevity research, scientists investigate whether mild, transient stress can stimulate endogenous repair networks to help preserve physiological function over time.
Research into hormesis spans several distinct experimental categories:
Preclinical results in cells or short-lived model organisms should never be confused with demonstrated human health outcomes. A compound or routine that extends the life of a roundworm under laboratory conditions does not constitute a verified human therapy. Translating laboratory observations into clinical practice requires rigorous human trials that measure validated endpoints over meaningful timeframes.
Traditional toxicology long relied on linear models of harm. In those older frameworks, any exposure to a damaging agent was assumed to create proportional risk. Hormesis challenges this linear view by demonstrating an inverted U-shaped or U-shaped curve, depending on the measured physiological outcome. At very low levels, an agent may stimulate repair pathways without causing lasting damage.
The peak stimulation observed in hormetic experiments is generally modest. Reviews across biological systems indicate that the adaptive response typically enhances baseline defense capacity by ten to thirty percent. It does not produce infinite biological enhancement. If the stressor intensity or duration increases beyond a critical threshold, the response shifts rapidly from adaptation to functional impairment.
Dose is not simply a single numerical quantity. In living organisms, dose consists of several interacting variables:
A stimulus that triggers robust adaptation in a well-rested adult can cause structural damage in someone who is sleep-deprived or malnourished. A single exposure might prompt beneficial cellular signaling. That same exposure, repeated daily without adequate rest, can produce chronic exhaustion of cellular reserves. Understanding the biology of aging and longevity science requires analyzing these recovery dynamics rather than assuming stress is inherently protective.
Living cells maintain an array of latent maintenance systems. Under normal, unperturbed conditions, these systems operate at a steady baseline rate to conserve energy. When a mild perturbation occurs, specialized molecular sensors detect the disturbance and recruit reserve capacities. This response is often framed as an expansion of homeodynamic stability.
Proteins perform the primary structural and catalytic work inside cells. Environmental stressors such as elevated temperature, oxidative shifts, and heavy metals can cause delicate protein chains to unfold. Unfolded proteins threaten cellular health because they can aggregate into toxic clumps.
When mild thermal or chemical stress occurs, cells upregulate heat-shock proteins. These molecular chaperones bind to misfolded protein chains and guide them back into their correct three-dimensional shapes. If a damaged protein cannot be refolded, the heat-shock system directs it to the proteasome or lysosome for degradation. This process maintains proteostasis, preventing the accumulation of nonfunctional proteins commonly
seen in aging tissues.
For decades, reactive oxygen species were viewed strictly as damaging metabolic byproducts. Classical theories of aging proposed that cumulative oxidative stress inexorably degraded cellular lipids, DNA, and proteins. Modern geroscience paints a far more nuanced picture of redox biology.
Mitochondria produce small amounts of reactive oxygen species during normal energy generation. When physical activity or temporary nutrient scarcity temporarily increases mitochondrial activity, reactive oxygen species rise briefly. Rather than causing catastrophic damage, these low-level oxidants function as critical signaling molecules. They oxidize specific cysteine residues on regulatory proteins, triggering genetic transcription programs that upregulate endogenous antioxidant enzymes like superoxide dismutase, catalase, and glutathione peroxidase.
This phenomenon, termed mitohormesis, demonstrates that completely eliminating reactive oxygen species can actually impair cellular defense readiness. The transient oxidant pulse acts as an informational cue. It signals the cell to strengthen its antioxidant shield before severe oxidative stress arrives.
Nutrient scarcity and metabolic challenges stimulate the cellular recycling program known as autophagy. During energy deprivation, cells activate AMP-activated protein kinase and suppress the mechanistic target of rapamycin pathway. This signaling shift prompts the cell to engulf worn-out organelles, dysfunctional mitochondria, and damaged protein complexes within double-membraned vesicles called autophagosomes.
These vesicles fuse with lysosomes, where acidic enzymes break the degraded components down into basic amino acids and fatty acids. The cell then reuses these raw materials for vital energy production and essential repairs. By clearing out defective cellular components, autophagy maintains quality control inside tissues. This recycling mechanism is a fundamental component of cellular health and metabolism.
Genomic integrity is constantly challenged by environmental radiation, metabolic toxins, and replication errors. Mild genotoxic stress can activate surveillance kinases like ATM and ATR. These enzymes initiate signaling cascades that pause the cell cycle, giving repair enzymes time to fix damaged DNA strands before replication occurs.
Similarly, mild exposures to dietary phytochemicals or environmental compounds activate the Nrf2 pathway. Under resting conditions, Nrf2 is kept in the cytoplasm by its inhibitor protein, Keap1. Mild electrophilic stress alters Keap1 structure, allowing Nrf2 to escape degradation and translocate into the cell nucleus. Once in the nucleus, Nrf2 binds to antioxidant response elements, initiating the transcription of Phase II detoxification enzymes that neutralize harmful chemicals.
Physical exercise serves as the most thoroughly documented human example of a hormetic stimulus. During muscular contraction, working tissues experience mechanical strain, localized energy depletion, elevated temperature, and an increase in reactive oxygen species. In isolation, each of these factors represents an acute biological stress.
The human body responds to this temporary disturbance through comprehensive physiological remodeling. Skeletal muscle fibers increase mitochondrial density, enhancing their capacity to generate cellular energy. Vascular endothelial cells adapt to increased fluid shear stress by synthesizing more nitric oxide synthase, which improves arterial flexibility and blood flow control. Systemic inflammation decreases in the days following exercise as tissues resolve the temporary inflammatory cascade required for muscle repair.
The signaling role of exercise-generated oxidants is clearly illustrated by human clinical trials involving high-dose antioxidant supplementation. Several controlled studies examined athletes taking large daily doses of synthetic vitamin C and vitamin E while undergoing endurance training. Researchers measured cellular markers of training adaptation, such as peroxisome proliferator-activated receptor gamma coactivator 1-alpha and citrate synthase activity.
In multiple trials, subjects receiving high doses of antioxidants exhibited blunted increases in mitochondrial biogenesis and insulin sensitivity compared to subjects taking a placebo. The exogenous antioxidants rapidly scavenged the exercise-induced reactive oxygen species, extinguishing the redox signals required to activate transcription factors for mitochondrial growth.
The clinical evidence regarding long-term athletic performance remains complex. While high-dose antioxidants consistently suppress specific cellular signaling cascades in skeletal muscle biopsies, their impact on gross performance metrics like race times or maximal oxygen uptake varies across studies. Nonetheless, these findings demonstrate that artificially eliminating physiological stress signals can interfere with endogenous adaptive responses.
Because moderate exercise improves cardiovascular and metabolic biomarkers, it is tempting to conclude that extreme volumes provide even greater health advantages. Epidemiological and clinical cardiology studies suggest that the dose-response relationship between exercise volume and health outcomes eventually reaches a plateau, and may follow a reverse-J shape for certain specific cardiac endpoints.
Large cohort studies examining leisure-time physical activity show that the greatest reduction in all-cause mortality occurs at approximately three to five times the standard public health recommendations. Beyond this volume, mortality risk remains significantly lower than that of sedentary individuals, but additional hours of intense exertion do not confer proportional life-extension advantages.
At extreme endurance volumes maintained over decades, a small subset of athletes demonstrates higher rates of coronary artery calcification, myocardial fibrosis, and atrial fibrillation compared to moderate exercisers. These findings do not indicate that heavy exercise is broadly dangerous. They simply show that the biological benefits of physical exertion follow a biphasic distribution rather than an infinite linear ascent.
Nutritional deprivation represents another major area of longevity research where hormetic principles are actively studied. In animal models ranging from yeast to rodents, reducing daily caloric intake without malnutrition reliably extends mean and maximum lifespan. Translating these findings to human physiology has required controlled clinical trials that evaluate intermediate markers of aging.
The Comprehensive Assessment of Long-term Effects of Reducing Intake of Energy Phase 2 trial represents the benchmark human study of dietary restriction. The trial enrolled 218 healthy, non-obese male and female volunteers between the ages of 21 and 51. Participants were randomized into two distinct groups for a duration of two years:
Achieving a substantial, continuous calorie deficit over two years in free-living human subjects presents significant behavioral hurdles. While the study protocol prescribed a 25 percent restriction, objective physiological measurements using doubly labeled water showed that participants achieved an average caloric reduction of 11.7 percent across the trial.
Researchers analyzed blood samples and physiological data from the CALERIE cohort to determine whether mild caloric restriction alters the rate of human biological aging. The trial yielded several meaningful intermediate findings:
The trial also evaluated biological age using advanced DNA methylation algorithms. Researchers compared changes across multiple epigenetic clocks to determine how caloric restriction affected the cellular aging rate.
The results differed depending on the specific computational clock applied. The intervention produced a statistically significant slowing of the pace of aging as measured by DunedinPACE, representing an estimated three percent deceleration compared to controls. Analyses using the PhenoAge and GrimAge biological age algorithms did not demonstrate statistically significant treatment-by-time differences between the groups.
These disparate results highlight an essential lesson in modern geroscience. Epigenetic clocks capture different aspects of cellular physiology and chronological time. A change in a single surrogate measurement does not prove that an individual will live longer. The CALERIE trial confirms that mild caloric challenge can improve metabolic and inflammatory risk factors in healthy humans, but it does not establish extended human lifespan.
Much of what is known about the genetics of stress resistance originates in laboratory model organisms. The roundworm Caenorhabditis elegans is widely used because its short two-week lifespan allows researchers to track survival curves across thousands of individuals.
In C. elegans, exposing young worms to mild, non-lethal heat stress or low concentrations of chemical pro-oxidants induces cross-tolerance. The conditioned worms survive subsequent, otherwise lethal thermal challenges far better than unconditioned controls. Furthermore, these mildly stressed worms often show extended mean lifespans.
Genetic knockout experiments reveal that this lifespan extension depends on specific molecular pathways:
Despite the elegance of these genetic discoveries, serious translational barriers prevent direct extrapolation to human health. Model organisms live in highly controlled, pathogen-free laboratory environments. In these sterile settings, an animal does not need to fight real-world infections, endure physical trauma, or perform complex cognitive tasks.
A genetic alteration that increases stress resistance in a roundworm often carries severe evolutionary fitness trade-offs. In natural environments, organisms that divert excessive metabolic resources toward continuous cellular defense frequently suffer from impaired fertility, decreased growth rates, and reduced physical vigor. Demonstrating that a stressor extends the life of an invertebrate under artificial laboratory conditions does not indicate that exposing humans to the same stressor will safely slow biological aging. For those interested in evidence-based strategies, exploring valid longevity interventions and therapeutics requires examining trials conducted directly in human subjects.
When evaluating scientific papers on hormesis and aging, it is critical to distinguish between different types of experimental endpoints. Many commercial health claims conflate acute survival during a stress test with true extension of healthy human life.
Researchers organize physiological outcomes into four distinct categories:
Evidence demonstrating an improvement in one category does not automatically imply improvements in the others. For example, a dietary compound may increase the expression of antioxidant enzymes in cultured fibroblasts without improving physical endurance in living animals. Similarly, an intervention that increases acute thermal resistance in nematodes may have zero impact on human cardiovascular disease risk.
Surrogate biomarkers provide valuable clues about biological mechanisms, but they are not equivalent to hard clinical endpoints. When reviewing studies on biological age testing, readers must remember that algorithms like DNA methylation clocks, blood chemistry panels, and physiological frailty indices measure computational approximations of biological state. They do not provide an exact forecast of future lifespan.
Applying biological stress to improve health involves distinct physiological hazards. If the intensity, duration, or frequency of a stressor exceeds an individual's adaptive capacity, the stimulus becomes explicitly destructive.
The capacity to mount an effective stress response declines as organisms grow older. In young, healthy tissues, molecular sensors rapidly detect homeostatic disruptions and initiate robust protective cascades. In aged tissues, this sensing and response machinery becomes sluggish and less coordinated.
A physical challenge that produces a beneficial adaptive response in an active thirty-year-old can cause tissue damage in an elderly individual with low physiological reserve. In older organisms:
For these reasons, hormetic interventions cannot be prescribed using universal protocols. A stimulus must be carefully matched to the baseline reserve capacity of the recipient. Exposing frail individuals to severe environmental or metabolic stress in the hope of rebuilding vitality can easily lead to catastrophic decompensation.
The benefit of a hormetic challenge is realized during the recovery phase, not during the acute stress exposure itself. When a muscle fiber is loaded during weight training, it experiences microscopic structural damage and glycogen depletion. The physical growth and mitochondrial adaptation occur during the subsequent hours and days of rest, proper nutrition, and restorative sleep.
If an organism is subjected to repeated physical challenges without sufficient recovery time, the homeostatic systems enter a state of chronic strain. Under conditions of inadequate rest:
True resilience requires balancing the challenging stimulus with an equal commitment to biological recovery. Without sufficient rest, supposed hormetic practices simply become chronic physiological damage.
Scientific integrity requires stating what the evidence on hormetic biology cannot support. Longevity science is frequently distorted by exaggerated marketing claims that misinterpret early laboratory data.
The published scientific literature does not support the following assertions:
Understanding the longevity science and healthspan research published by reputable academic institutions enables individuals to evaluate emerging claims with appropriate scientific caution.
To help readers navigate the scientific literature, the following definitions clarify terms frequently encountered in research on stress response and aging.
Translating the principles of hormesis into daily life requires focusing on well-established, recoverable lifestyle practices. Readers who want to support their physiological resilience can apply the following checklist:
Stay current with research on aging biology, biomarkers, nutrition, therapeutics, peptides and longevity technology. AgeAmaze reports what the evidence shows, where uncertainty remains and which claims still need stronger data.


Follow AgeAmaze for careful reporting on what longevity science can show today and what still needs stronger evidence.
read the Blog