A gene-expression screen identified SRSF1 as an aging research candidate. Examine the fibroblast findings, mouse results and limits of the evidence.


On 2026-10-15, Technology Networks covered an aging study led by George Church’s group at the Wyss Institute at Harvard University. The paper, “Transcriptomic reprogramming screen identifies SRSF1 as a regulator of aging,” appeared in Nature Aging in 2026.
The researchers identified SRSF1 as the leading candidate in a gene-overexpression screen designed to shift aging-associated patterns in human fibroblasts. They reported changes in several cellular aging features, while the Wyss Institute reported slower frailty progression and a 14% increase in median lifespan compared with controls in aged mice. The central finding is a preclinical proof of concept: a gene-expression model helped identify a candidate that could then be examined through cellular measurements and animal outcomes.
Study setting: In vitro experiments using cultured human fibroblasts and animal experiments in aged mice, not a human therapeutic trial.
According to Technology Networks, the researchers trained their machine-learning transcriptomic aging model on gene-expression data from 464 fibroblast samples. The samples came from donors spanning a wide age range. The model estimated transcriptomic age and supplied a readout for assessing whether experimental interventions shifted expression patterns toward a younger profile.
Here, “transcriptomic age” refers to an estimate based on gene-expression patterns. The model compares those patterns with age-associated relationships represented in its training data. Researchers could then use its output to score changes after an intervention, rather than relying only on a visual impression of the cells.
Technology Networks reports that the predictor detected transcriptomic-age shifts in three fibroblast cell lines from donors aged 55, 65, and 79. The experimental interventions included Yamanaka factors. This part of the work examined whether the model registered changes after interventions intended to alter cellular state.
The study then paired this measurement approach with a gene-overexpression screen. The clock supplied a signal for comparing candidates, while the screen tested which genes shifted that signal. SRSF1 emerged as the leading candidate for follow-up experiments.
That sequence matters for interpreting the work. Building an age predictor and identifying an intervention are separate research tasks, even when they are combined in one platform. The predictor provides a way to rank experimental changes; subsequent experiments examine what those changes involve biologically.
Readers comparing this approach with other aging measurements may find it useful to distinguish the signals different biological-age models measure. In this study, gene expression was both the basis of the age estimate and a central target of the experimental screen.
SRSF1 is an RNA-processing and splicing factor. According to the study coverage, increasing its expression was associated with changes across several aging-related features in fibroblasts. The findings therefore extended beyond a shift in the transcriptomic-age estimate alone.
The researchers reported reduced cellular senescence, inflammatory signaling and proteostatic stress. They also reported restoration of DNA-repair programs. Together, these observations connected the screening result with several cellular processes relevant to the study’s aging framework.
These were distinct measurements rather than interchangeable descriptions of the same result. A younger-looking expression profile was the screening signal. The observations involving senescence and cellular stress provided additional biological context for that signal, while the DNA-repair findings pointed to another program affected in the experiments.
The treated cells also retained fibroblast morphology and function-associated gene expression. They did not activate the pluripotency programs associated with Yamanaka factors in the reported experiments. That distinction placed cell identity alongside age-associated expression as an important feature of the follow-up work.
The Wyss Institute account quotes co-first author Alex Plesa describing “a fundamental tradeoff between rejuvenation and cell identity.” The SRSF1 experiments addressed that tension by examining whether aging-associated features could shift while the cells retained characteristics of their specialized state. The relevant observation was preservation of fibroblast features under the conditions tested.
This gives the study a more specific biological question than whether a cell simply received a younger score. The question becomes which expression changes accompany alterations in cellular stress and repair, and how those changes relate to the cell’s existing identity. SRSF1 provided an experimental candidate through which the researchers could investigate those relationships.
The Wyss Institute reports that the researchers delivered SRSF1 to aged mice using a liver-tropic adeno-associated virus. The delivered material primarily accumulated in the liver. The animal experiment therefore examined a liver-directed intervention rather than uniform delivery throughout the body.
The mouse work brought survival and frailty into the assessment. Those outcomes address a different level of biology from a transcriptomic score in cultured cells. They allowed the researchers to examine whether the selected candidate was associated with outcomes in an aging animal.
The distinction between these experimental stages is important. The fibroblast model supplied the screening readout, cellular experiments examined associated biological changes and the mouse experiment assessed organism-level outcomes. Each stage contributed a different kind of evidence to the overall study.
The reported liver accumulation also makes tissue targeting central to interpreting the animal work. Where an intervention reaches is part of the experimental design, not a detail that can be separated from the result. Any account of the mouse findings should preserve that connection between delivery and outcome.
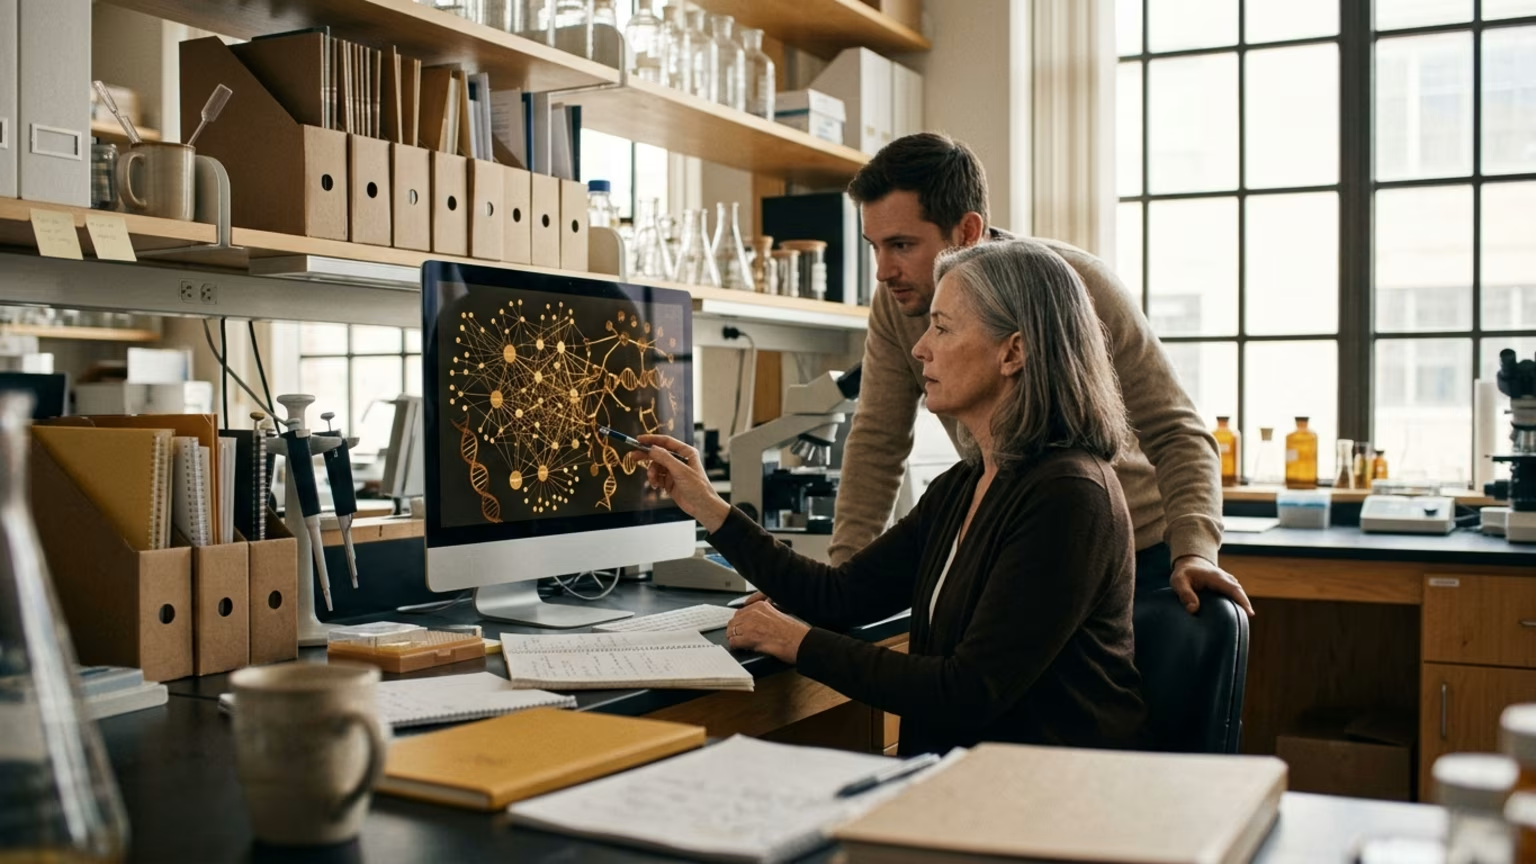
For a broader conceptual framework, it helps to view aging pathways as an interconnected biological map. This study linked an RNA-processing candidate with several cellular features and then examined outcomes at the animal level.
The study supports further investigation of SRSF1, but several boundaries determine how its findings should be read:
The practical reading rule is to identify the measurement and experimental setting before accepting a claim about rejuvenation. Ask whether the claim concerns a molecular score, a cellular feature or an animal outcome. Keeping those categories separate makes the evidence easier to judge without dismissing a potentially useful research lead.
For commercial testing claims, the relevant question is whether a biomarker has demonstrated usefulness for health decisions. Readers considering a test or intervention for personal use should discuss its intended purpose and supporting evidence with a qualified clinician.
The next phase should independently replicate the findings, connect SRSF1-associated splicing changes with functional outcomes and establish long-term safety under controlled tissue-specific delivery before moving toward human therapeutic evaluation.
Promoting an RNA-splicing candidate directly from a laboratory screen to a longevity treatment skips the evidence needed between those stages. AgeAmaze puts the underlying longevity biology into accessible language and keeps evidence strength visible, giving skeptical readers context for judging claims about biological age and emerging therapies.
Stay current with research on aging biology, biomarkers, nutrition, therapeutics, peptides and longevity technology. AgeAmaze reports what the evidence shows, where uncertainty remains and which claims still need stronger data.




Follow AgeAmaze for careful reporting on what longevity science can show today and what still needs stronger evidence.
read the Blog